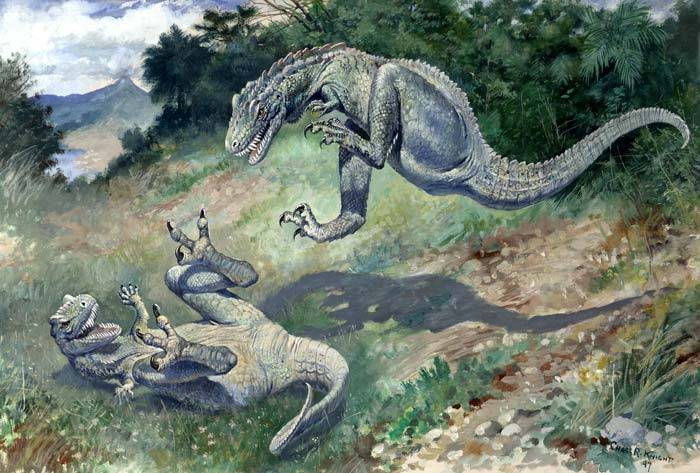Showing posts with label art. Show all posts

Wednesday, April 12, 2017

You're Doing It Wrong: Pteranodon Bills

Your bill's looking a little puny, there, buddy.
(Painting by Heinrich Harder, 1912, public domain).
Everybody knows Pteranodon. Quick, stop to imagine it! It's easy, because it's the most often-illustrated and well known pterosaur to the general public (though today's marketing departments often call it a pterodactyl, following it's original, century-out-of-date classification).

But hold on. That image you have in your head right now, of a big pterosaur with a long crest and a mid-length pointy beak? That's likely wrong, and may be just as much a hybrid as those Flintstones-style creatures with pteranodont crests and Rhamphorhynchus tails.

How do we know? Let's talk about Dawndraco.

Saturday, May 28, 2016

You're Doing It Wrong: Microraptor Tails and Mini-Wings

Type specimen of Zhenyuanlong, doing its best Archaeopteryx impression.
Just a short PSA today, and once again, it's about a paleoart meme that has outstayed its welcome.

Microraptor was the first time we got a good look at the feather pattern of dromaeosaurids. This is a big problem for two reasons. One, microraptors were small. That means that artists who were looking at them to extrapolate for bigger, more famous "raptors" could easily and somewhat justifiably write off their huge wings as a product of their size. Sure, we thought, microraptors had big wings, but they're tiny animals. Surely the bigger, more terrestrial dromaeosaurids didn't need such big wings. They probably still had wings, but they'd be smaller. Why would Velociraptor need such proportionately huge wings if it couldn't fly or glide?

Meme number two: that tail. I admit to being one of the first to go overboard when I fell, head over heels, for the "puff tailed dromeosaur" fossil (now the holotype of Cryptovolans, a synonym or close relative of the Microraptor) back around 2000. This was the first evidence we had of the tail feather style in dromeosaurids (or evidence that they even had remixes and rectrices at all. Remember When Dinosaurs Ruled America? That was plausible at the time it was being made). Naturally, having Microraptor plus Caudipteryx showed that the ancestral condition of pennaraptorans was a fan of feathers at the tip of the tail, not a fuzzy Sinosauropteryx like tail or a fully-vaned Archaeopteryx like tail. So artists ever since have been drawing dromeosaurids and troodontids and oviraptorosaurs with microraptor tails.

But that turned out to be wrong! It's an accident of history. We're now learning that Microraptor and Caudipteryx are weirdos.

Sunday, May 1, 2016

The First Feathered Dinosaurs (In Art)

The first illustration of a hypothetical "pro-avis" by Pycraft, 1906
Feathered non-avialan dinosaurs seem commonplace now, and it's hard to believe that there was a time, in living memory for some of us, when they were purely speculative. It makes sense, of course: once scientists realized (then realized again) that dinosaurs were the closest fossil relatives of birds, it was only natural to suggest that feathers had appeared in dinosaurs before they showed up in birds. To have a new type of animal, like Archaeopteryx, appear more or less fully formed with flight and feathers occurring simultaneously makes little sense in terms of evolution. Obviously, even if Archaeopteryx was considered the "first bird" or could fly in some rudimentary manner, it couldn't have been the first animal with feathers or feather-like integument. Feather-like structures had to have been present in the archaeopteryx's closest relatives. But what were those? For most of the 20th century, the answer would not have been dinosaurs.

Nopcsa's 1907 feathered, Compsognathus-like
"pro-avis" model at the Grant Museum, London.
Speculative bird ancestors with feathers or feather-like scales had been hypothesized and illustrated long before the first true feathered dinosaurs appeared in paleoart. These hypothetical "pro-aves", as they were generally termed, were first imagined by William Pycraft in 1906. Pro-aves were usually considered arboreal, gliding animals with elongated, feather-like scales, and Pycraft's illustration provided the template followed by many later illustrators, like Heilmann's 1916 version, and Burian's gorgeous but even more lizard-like 1960 rendition. Not all pro-avis illustrations followed this template, though. In 1907, Baron Nopcsa invented his own pro-avis, illustrating his hypothesis of a running, "ground-up" origin of bird flight. In addition to his illustration, Nopcsa created a wax model. Nopcsa thought birds might have evolved from quadrupedal reptiles which became more and more bipedal as their running speed increased, passing through a phase similar to Compsognathus, though not necessarily dinosaurian.

Beebe's "tetrapteryx", 1915.
There were also creatures like the "tetrapteryx", a speculative stage in the evolution of avian flight proposed by William Beebe in 1915. Beebe illustrated an Archaeopteryx-like creature with smaller wings as well as hind wings on splayed legs, reminiscent of early (but incorrect) illustrations of Microraptor. Other than the posture, the general anatomy of this hypothetical creature ended up being prescient by accident. His rationale for this hypothesis was the observation that some bird embryos develop and then lose feather quills on their legs. Heilmann, however, rejected this hypothesis after failing to find evidence among other bird embryos. New evidence to support this hypothesis was discovered in species like Microraptor, Anchiornis, and Sapeornis, which had various degrees of airfoils present on their hind legs, a line of evidence independent of the one supposed by Beebe. Though dinosaur-like in appearance, both Beebe and Heilmann considered the ancestors of birds to be "thecodont" grade archosaurs, not dinosaurs, so these hypothetical feathered thecodonts predated the first feathered dinosaurs in art.
Speculative reconstruction of a Triassic "carnavian" dinosaur
leaving feather traces in its trackway, from Ellenberger 1974.

The thecodont origin of birds did not truly give way to a dinosaur origin until the 1970s, after John Ostrom described the similarities between Archaeopteryx and Deinonychus. If dinosaurs were the new closest relatives of birds, then at least the most bird-like among them should be depicted with feathers (Ostrom himself disagreed with this though, and, according to Bakker, he fought the idea that Deinonychus should be feathered). Of course, which dinosaurs were most closely related to birds, and just how much of a gap remained between them and Archaeopteryx, allowed for considerable wiggle room and speculation.

A "carnavian" track maker
parachuting, from Ellenberger 1974.
In 1974, Ellenberger identified what he considered to be trace evidence for feathered dinosaurs from Lesotho, in the form of possible feather imprints and footprints which could have been made by small animals parachuting from trees, dragging their tail feathers in mud, etc. He illustrated a small bipedal dinosaur with feathers in the accompanying paper, along with totally speculative skeletal restoration of a new type of animal, nested within theropod dinosaurs, which he called "carnavians." Molnar, in 1985, dismissed the suggestion that these were feather imprints. Still, Ellenberger had become the first person to ever illustrate a non-avialan dinosaur, however hypothetical the species, with feathers.

Landry's influential 1975 restoration of "Syntarsus".
The next year, in 1975, a more famous feathered dinosaur illustration of a much better-known species was provided by Sarah B. Landry, drawn under the direction of Bob Bakker for his seminal article in Scientific American, "The Dinosaur Renaissance." Landry and Bakker depicted the small theropod "Syntarsus" (=Coelophysis) covered in overlapping feather-like scales or scale-like feathers, similar to Heilmann's "proavis", and a long tuft of feathers on the head. The choice of species was not a coincidence. Michael Raath, who had described Syntarsus in 1969 (the same year as Deinonychus), was quick to tout how bird-like it was in popular books and articles, and he suggested several times that it may have been feathered.

"Syntarsus" by Stout, 1976.

To understand the impact of this "first" feathered dinosaur, just look at the rest of the 1970s and early 1980s. It was Syntarsus, not Deinonychus, which was consistently drawn with feathers from then on. Many of these later reconstructions even directly aped Bakker and Landry's style of feather crest (or slightly modified it), making "Syntarsus with feather crest" a bona fide paleoart meme. Many of these left out the more subtle body feathers of the original, unfortunately, possibly influencing decades of "half-arsed" theropods with feather mohawks, up to including the dinosaurs in the 2001 film Jurassic Park III more than 20 years later. (One notable exception to the Syntarsus trend was also a watershed moment for paleoart. After reading Bakker's article, a paleoartist named Gregory S. Paul drew his first feathered dinosaur: an Allosaurus).

One of my favorite derivatives of Landry's Syntarsus illustration is one made in 1976 by William Stout and reproduced in Don Glut's 1982 edition of The New Dinosaur Dictionary. Though Glut pointed out that the feathers were speculative, they're probably less inaccurate than the legless snake it's eating! Also included in Glut's revised dictionary was one of the first illustrations of the theropod Kakuru, by Mark Hallett. Though just as speculative as Ellenberger's drawing (Kakuru is known only from two limb bones), it has more of a modern feel. The reclining theropod is decked out in long, filamentous feathers, rather than the broad, scale-like feathers of Landry's Syntarsus. It's worth noting that all of these early drawings of feathered dinosaurs had bare or scaly faces. This method of emphasizing the transitional character of early feathered theropods was probably inspired by traditional portrayals of Archaeopteryx, a "bird" with the head of a "reptile."

Feathered ornithischians, by Lorene Bjorklund, from
The Warm-Blooded Dinosaurs, 1979.
Many bird-like dinosaurs actually had feathers covering some or all of the face as well as the body, though some kind of "modular evolution" did occur to a degree in a few lineages (here's looking' at you, Darwinopterus). And some Mesozoic dinosaurs, most famously Kulindadromeus, seem to have feathers restricted to certain body segments with abrupt transitions between feathery and scaly regions. So, this much-maligned meme isn't necessarily out of the question, at least in early feathered lineages.

A few very early books featuring extremely prescient feathered dinosaurs came in 1978 and 1979. First, Julian May brought us perhaps the first renaissance-era dinosaur book for kids, The Warm-Blooded Dinosaurs, which featured not only a feathered Struthiomimus by Lorene Bjorklund on the cover, but several feathered ornithischians inside. An Iguanodon looks sort of ambiguously feathered (it might just be the crosshatched style), and interestingly, has a abrupt transition to a croc-scutes tail very similar to Kulindadromeus. There's also a skeletal of Microvenator with a fuzzy, Greg Paul style silhouette outline. The next year, Archosauria: A New Look at the Old Dinosaur by John McLoughlin includes some species with feathered faces for the first time, like his amazing, feathered Coelurus. It's odd as a modern reader to see that in both of these books, it's the more basal dinosaurs shown with feathers. Primitive ornithopods and "coelurosaurs" (considered a paraphyletic grade of early, ancestral dinosaurs at the time) like Syntarsus, Coelurus, and Saltopus are given feathers while deinonychosaurs like Saurornithoides and Deinonychus are not. The influence of the thecodont theory was still going strong, with birds thought to have evolved from the earliest dinosaurs rather than deinonychosaurs, which were exclusively known from the Cretaceous at that time.

Kakuru by Mark Hallett, from Glut 1982.

Ironically, Deinonychus, which out of all these dinosaurs was most similar to Archaeopteryx, did not become consistently or even frequently depicted with feathers until the at least the late 1980s. This was also probably due, in part, to artistic inertia. The original illustration of Deinonychus that accompanied Ostrom's description was so iconic that it was being copied well into the '90s. One of the first depictions of a feathered Deinonychus was a statuette produced by sculptor and founding father of Neopaganism Otter Zell (aka Oberon Zell). If anybody who owns a copy of this statuette wants to trade it for my right arm, please let me know.

After Syntarsus, the next non-avialan to become consistently depicted with feathers was Avimimus. From its first discovery, Avimimus was interpreted (and in some cases, like the supposed lack of a tail, misinterpreted) as being as birdlike or more than Archaeopteryx. Though commonly misreported online as having quill knobs, Avimimus actually had a flat ridge on the ulna which has been interpreted as a similar kind of support for the soft tissue of a feathered wing. Though not the same kind of direct evidence as quill knobs would be, most paleoartists ran with the suggestion, and most early Avimimus illustrations did portray it with feathers. John Sibbick restored it that way for David Norman's 1985 Illustrated Encyclopedia of Dinosaurs, and his version is a down-right throwback to the "pro-aves" of the early 1900s, with long, scale-like feathers on the outstretched arms and tail.
The first(?) feathered Deinonychus,
a statuette by Otter Zell, 1984.

1986 saw the publication of Bakker's The Dinosaur Heresies, filled with his own illustrations of feathered dinosaurs, including Deinonychus. (Stout and Paul had both continued to illustrate feathered dinosaurs up to this time, though not all were published or widely distributed at the time). Bakker's book opened up the door to more mainstream portrayals of this controversial subject, and it's no coincidence that many other artists were working the occasional feathered dinos into books and articles in the years that followed. Most notable among these were Paul's Predatory Dinosaurs of the World in 1988, and children's books inspired by it like The News About Dinosaurs. From then on, every "renaissance" era dinosaur book worth its salt included at least one speculative feathered theropod. Some books were bold enough to become the first to put "Feathers On Bloody Everything" (to quote the lament of some current-day feather detractors), theropods and ornithischians alike, as in 1988's speculative evolution book The New Dinosaurs by Dougal Dixon.

Two early restorations of Avimimus. Left: by Sergai Kurzanov, looking very bird-y.
Right: By John Sibbick from Norman's Encyclopedia, looking very much like Heilmann's "pro-avis."
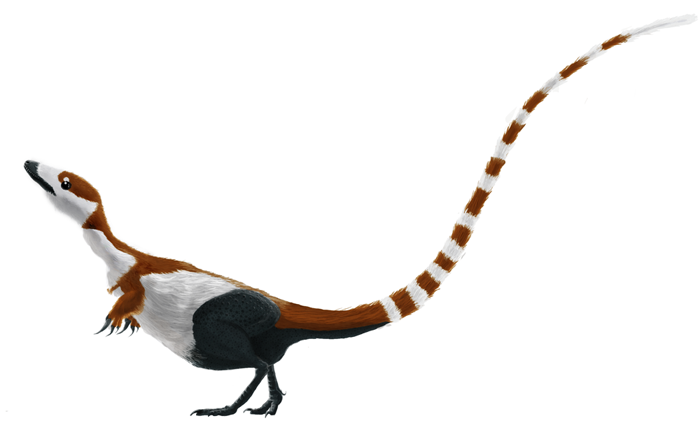
By the time the first actual feathered dinosaur was announced in 1996, dinosaur fans, if not the general public, had been well prepared and had even come to expect such a find to be inevitable. The fact that this first find was Sinosauropteryx unfortunately reinforced some stereotypes that had been perpetuated by early renaissance era paleoart, such as short, fur-like feathers, naked legs and bellied, and half-feathered faces. Paul essentially invented the latter meme in an attempt to make his theropods look more bird like (by suggesting a sort of beak), and while this was his own personal speculation, many later artists ran with it, including in early drawings of Sinosauropteryx. The fossil appeared to support the hypothesis, which would have been an incredibly lucky guess for Paul if not for the fact that the snout past the eyes on that specimen had not even been fully prepared out of the rock (maybe, just maybe, because the scientists themselves were so influenced by Paul that they didn't expect any feathers to be found there!).

A modern feathered dinosaur:
 Tianyulong sculpture by Jason Brougham, 2016.
In a way, modern paleoart is still struggling to shed the memes and conventions generated by this pre-evidence feathered dinosaur artwork. Many artists are starting to critically examine just how far-off much of that early art really was, and to realize that it was, of course, just pure speculation about what may be, not informed speculation based on fossil evidence. Many dinosaurs, especially non-avialan coelurosaurs, had a feather covering that was much more Archaeopteryx-like than any of those pioneering artists could imagine. It's only recently that many of the best artists have been going back for inspiration not to Landry and Paul and Bakker, but to the earlier artists who were drawing Archaeopteryx and the various "pro-aves". This new era of paleoart, part of what Tom Holtz has dubbed the "Dinosaur Enlightenment," will no doubt generate its own set of tropes which will need to be overcome by the next generation of artists. We're already seeing that with the dogmatic insistence from some quarters on a certain standard of feathering for all dinosaurs when the fossils are starting to suggest much more variety. With any luck, the internet will allow this new generation to push forward and more widely and rapidly share new ideas and possibilities about what feathered dinosaurs can be.

Friday, April 10, 2015

The Brontosaurus Club

Brontosaurus excelsus - the triumphant return.
By M. Martyniuk, all rights reserved.
By now, anybody who's interested in paleontology, and their mother, and their great uncle, have probably heard the news: Brontosaurus is back!

Of course, the more technically minded paleo fans will know that Brontosaurus never actually went anywhere. Ever since its first specimen was studied in 1879 by Bone Warrior O.C. Marsh, paleontologists have agreed that the species Brontosaurus excelsus* was unique among sauropods. The question soon became, however, exactly how unique. In 1903, Elmer Riggs decided that it was similar enough to another sauropod species, Apatosaurus ajax, that they should both be placed in the same category of sauropods, and since Apatosaurus was an older category ("genus") name than Brontosaurus, he reclassified the species as Apatosaurus excelsus. However, it was clear even to Riggs that Apatosaurus excelsus and Apatosaurus ajax were different species, and the decision to "lump" them together into one category was always subjective and non-scientific - these kinds of things are a matter of taste only.

Saturday, February 21, 2015

The Evolving View of Stegosaurus

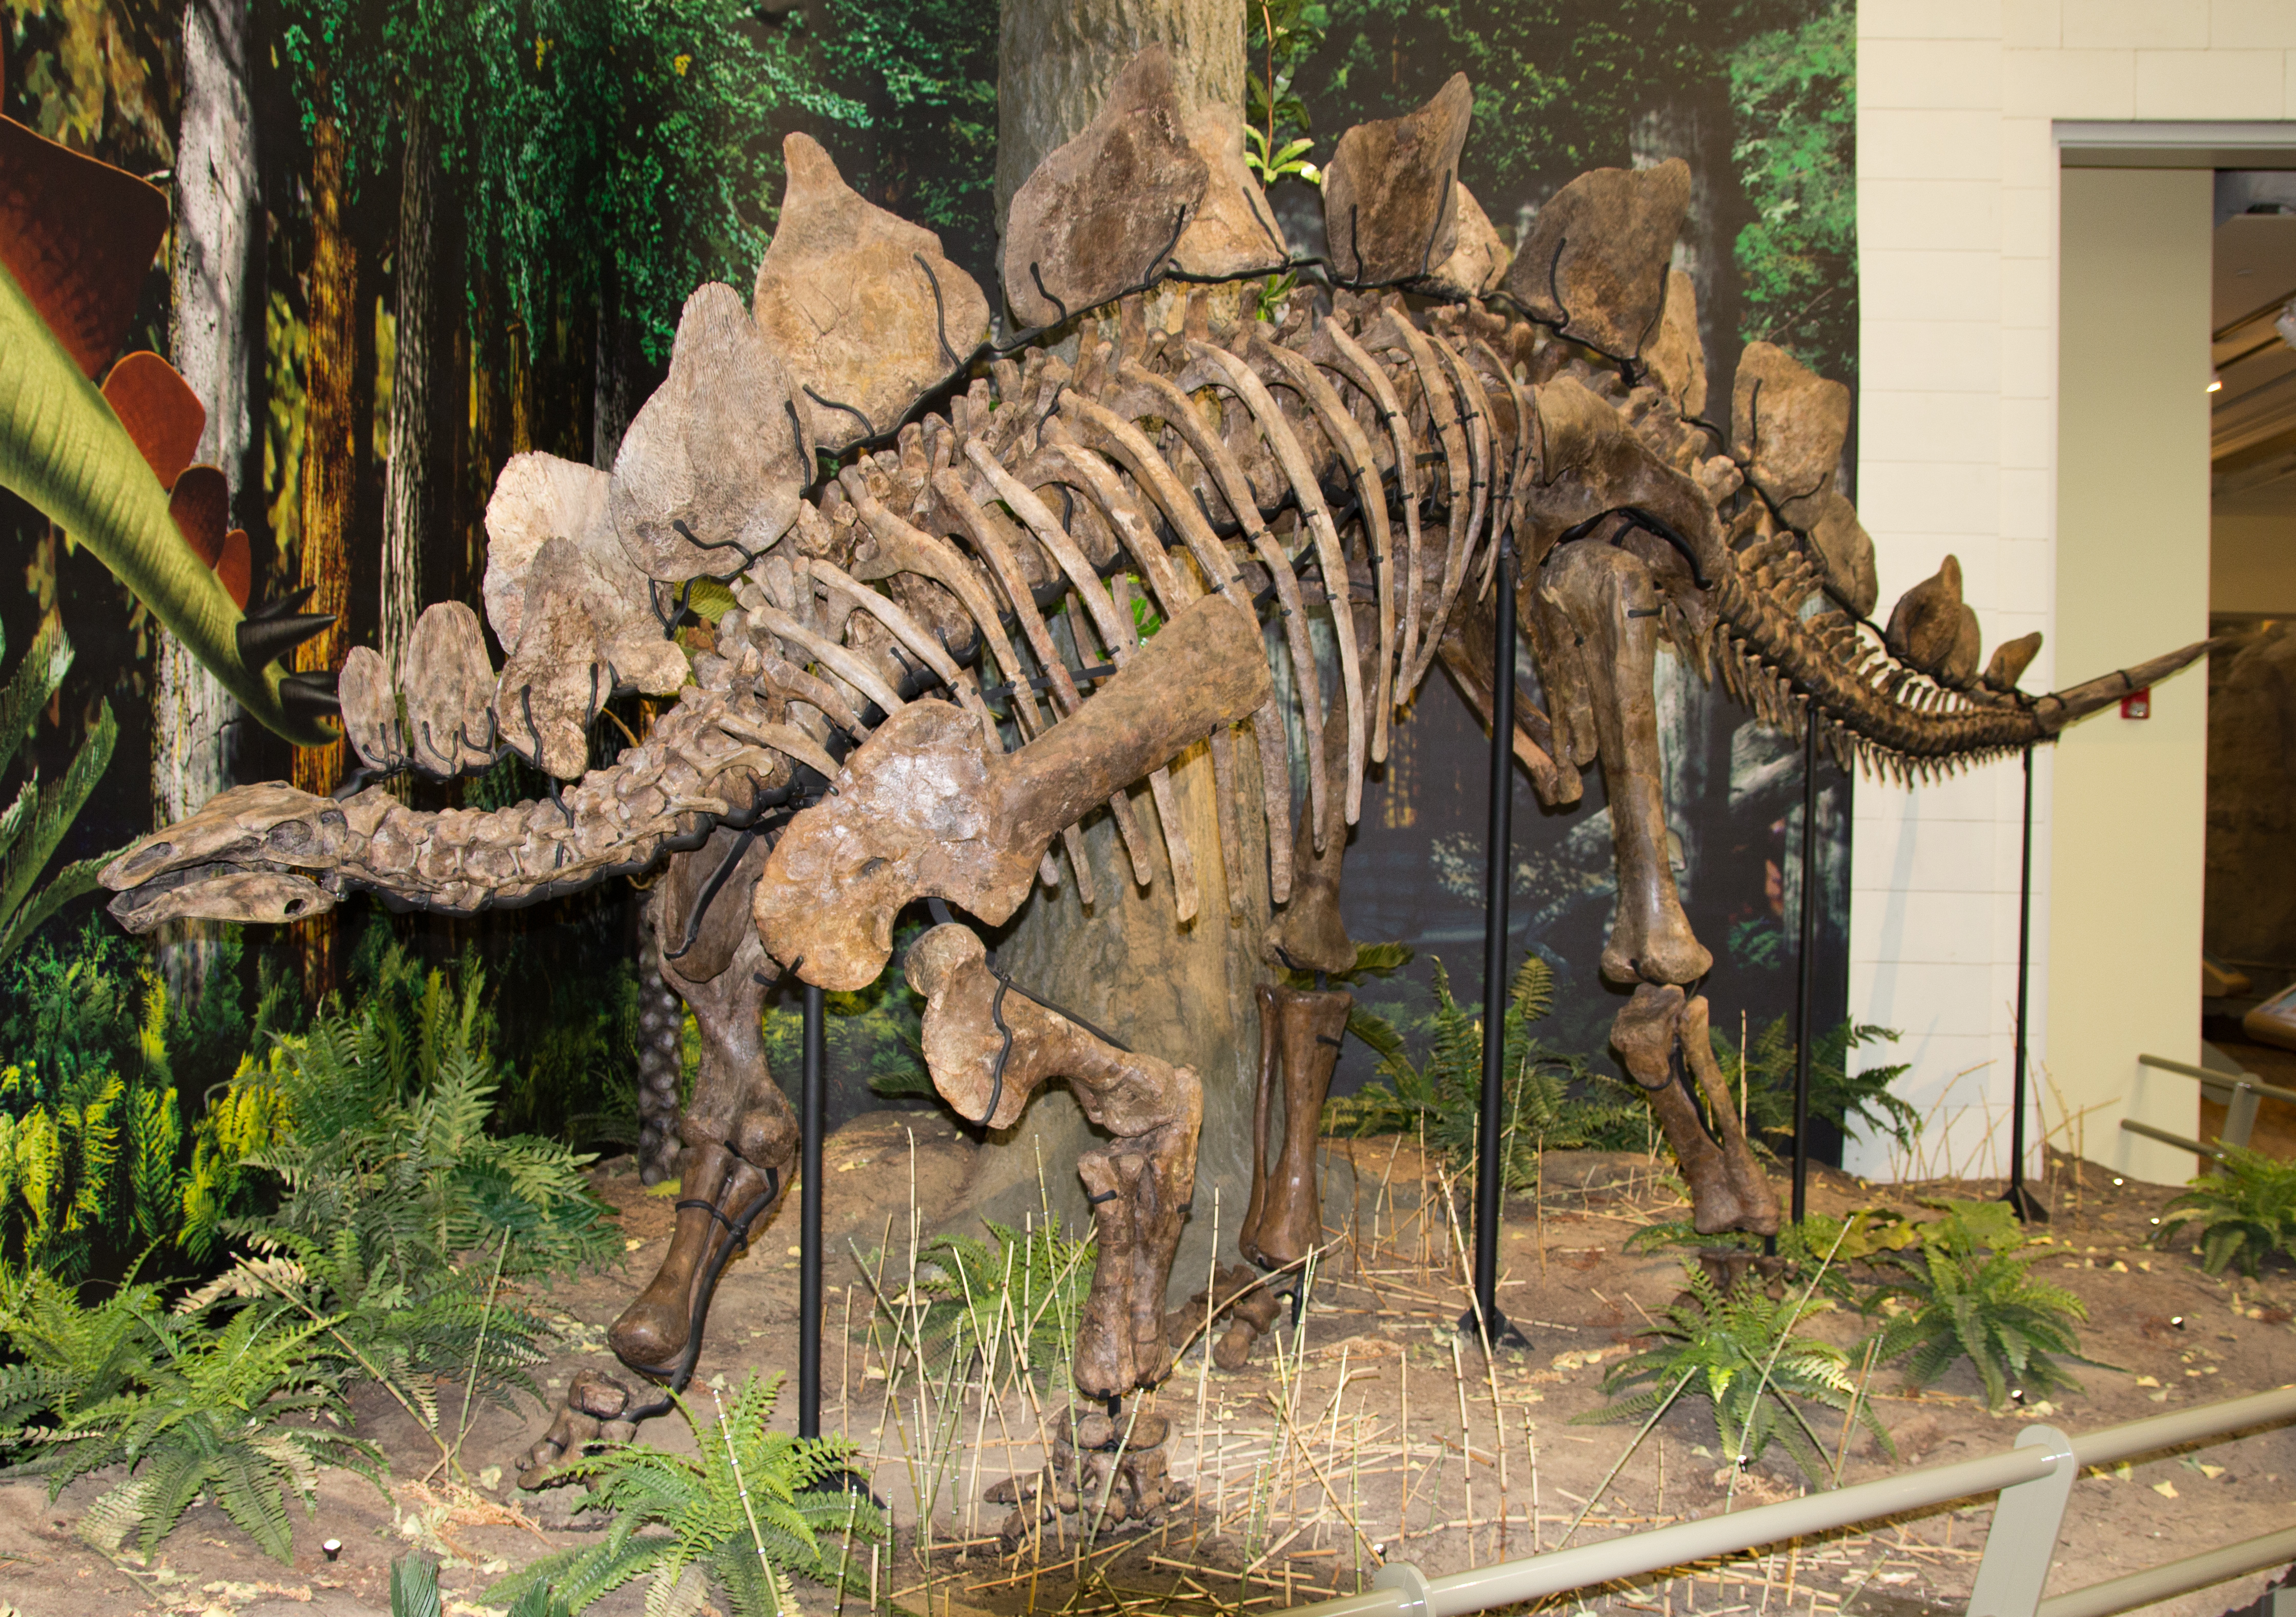
Mounted skeleton of Stegosaurus ungulatus at the Carnegie Museum. The tail, plate, and spike arrangement have been updated in this mount to reflect current thinking following the study by Carpenter (1998). Photo by Perry Quan, CC-By-SA 2.0.
Seeing as how I've been working on restorations of two different stegosaur species this month, I thought I'd write up a quick review of the most famous aspect of these iconic dinosaurs: Their big, triangular plates. For a complete overview of the history and interpretation of Stegosaurus, be sure to see Ken Carpenter's 1998 paper.

Interpretation of the life appearance of stegosaurs has changed several times since they were discovered by O.C. Marsh in 1877. The first stegosaur fossil (belonging to the species S. armatus) were found near the town of Morrison, Colorado, but the specimen was disarticulated and only a few of the plates were preserved. Initially, Marsh thought that these plates played flat along the animal's back, forming a sort of turtle-like shell, or like the tiles on a roof (hence the name Stegosaurus, which means "roofed lizard"). Marsh also initially believed that stegosaurs were aquatic, due to this turtle-like appearance, but also that they would have walked on two legs on land.

Sunday, November 30, 2014

Is Jurassic World Stealing from Independent Illustrators?

Sorry for the clickbait title. The answer is yes. Yes they are.

It's one thing when toy companies do it.

It's quite another when a big-budget Hollywood movie starts stealing the work of independent paleoartists and illustrators for use in their production design.

It started when well-known paleo illustrator Brian Choo posted the following modified production still to his DeviantArt account. The photo in question is fairly low res and comes from the newly opened Jurassic World web site. The still features children using a prop in the movie called a "Holoscape", presumably a kind of interactive computer terminal featuring information about the various kinds of dinosaurs in the park.


Saturday, October 11, 2014

You're Doing It Wrong: Protobird Toys Edition

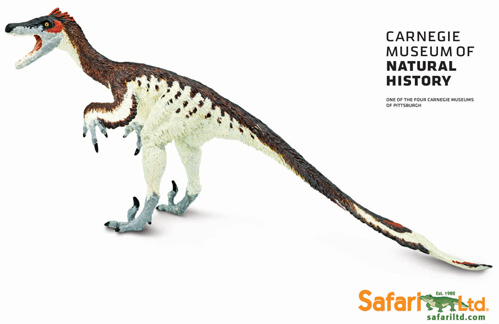
The new Carnegie Velociraptor figure.
I'm pretty slack when it comes to keeping up with my Twitter account, but if one thing can get me to break my one post per month general rule, it's "somebody is wrong on the Internet!" Or, in this case, "somebody made an inaccurate dinosaur model under the auspices of museum-approved accuracy!"

Let me preface this post with a few disclaimers. One, I have no problem with people making dinosaur art however they like. But I feel it's very important to draw a distinction between dinosaur art in general and paleoart. Creating a drawing, painting, or sculpture under the guise of paleoart implies that some degree of research went into the piece. When evaluating paleoart, critics are completely entitled to demand as rigorous an approach to accuracy as the evidence allows. Of course, speculation must be included to some degree, but the baseline expectation is always that basic facts and plausible inference will be taken into consideration.

Dinosaur art is a for of pop art, a purely artistic expression. Paleoart is a representation of a scientific hypothesis about the life appearance and behavior of an extinct organism.

This recent Twitter kerfuffle was due specifically to the debut of a new dinosaur figure in the Carnegie Collection produced by Safari Ltd. I've been a big fan of the Carnegie figures (and the sometimes nicer quality Wild Safari sister series) since I was a wee lad buying my first Carnegie Pteranodon in a little hobby shop for about $2, and pining over their massive Brachiosaurus. Carnegie figures have obvious appeal for scientifically-minded young dinosaur fans. First, most of them are made with a consistent scale (usually 1:40), so when you line them all up you can see how big each animal was compared to one another. Second, they are marketed as having the highest level of scientific authority: the Carnegie Museum stamp and assurances that hey are approved by actual paleontologists gives them the weight of authority and accuracy not found in many other toy lines. Sure, many of the older figures, including my Pteranodon, are now sorely out of date, but this is due largely to the Science Marches On effect rather than a basic, original inaccuracy.

However, like many paleoartists, the sculptors at Carnegie and related accuracy-minded/marketed toy lines seem to be having, well, let's say a little trouble adapting to the feathered revolution. Trained in the '80s and '90s drawing and sculpting Paulian, reptilian dinosaurs, it's been a steep learning curve for many of these artists to switch to bird-like, feathered dinosaurs, which many artists don't even realize requires a crash course in avian anatomy, rather than reptile or mammal anatomy, to get right. This is why expert consultants are so important in these projects--artists simply need help catching up with the latest research. Unfortunately, they're usually getting bad advice from "experts" who simply do not care.

The newest entry in the Carnegie Collection is the old favorite Velociraptor. Carnegie had previously released a scaly Velociraptor, but like many of their other models, they have commendably updated it to try and reflect current science. Unfortunately, it seems they mainly achieved this by slapping feathers over the basic original model with no regard for the fact that feathers inherently change the entire presentation and outline of an animal. Unlike fur or "protofeathers", which just fluff up the outline of an animal, feathers are more like a mobile exoskeleton that re-defines the entire body.

My own hypothesis, based on fossil and phylogenetic evidence as well as
inference from living analogues, about the life appearance of Velociraptor.
That being said, the Carnegie Velociraptor is not that bad overall and is very nicely sculpted, with an interesting and plausible color scheme. The feathers look fur-like, true, but this is not unprecedented among different lineages of large ground birds, and so is not unlikely in flightless protobirds (though they'd probably still be longer). The main problem here is the wing. Yes, wing. Like chickens and ostriches, protobirds possessed fully-fledged wings despite being flightless or nearly so, and retaining large claws on the fingers (yes, chickens, ostriches, and many other birds have hand claws--they are not some prehistoric protobird relic!).

Specifically, the wings in the new Velociraptor figure are very small, with short feathers, and are present only on the forearm, not the hand, making them only half a wing--literally, since they're issuing the primary feathers. We do not have direct evidence of primaries, but we have never found a single example of a maniraptoran that has secondaries but not primaries, and so it should be assumed they were there by default. As for secondaries, we have direct evidence in the form of quill knobs for this species. Quill knobs are not found in all feathered animals, let alone all flying birds, and seem to be associated with strong attachment either due to high-stresses during flight or other flapping behavior and/or especially large/long individual feathers.

Long story short: Not only did Velociraptor have wings, it probably had larger wings than many other dromaeosaurids. AFAIK not even Microraptor and Archaeopteryx had quill knobs to support their wings.

The new Carnegie figure, on the other hand, barely has wings at all. What went wrong?

Some insight can be gained by a recent series of incidents involving sculptor Dan LoRusso on the message board of the Dinosaur Toy Blog. LoRusso Is an amazing artist and is responsible for some of my all-time favorite dinosaur figures released in the Boston Museum of Science Collection by Battat (now being re-released with updates and new figures under the Terra brand). Collectors were understandably excited about the fact that the Battat series was coming back after nearly two decades, though the excitement was dampened a little by some obvious accuracy issues in the new figures, specifically when it came to the feathered species (or species that should have been feathered).

LoRusso was criticized online for producing a very well done but very inaccurate therizinosaur figure which completely lacked feathers. It would have fit right in with the excellent quality and Paulian style of the original series... back in 1994. But in 2014, when we have incontrovertible proof that therizinosaurs were not only feathered but that at least smaller species were very densely feathered, it is simply bizarre to see a featherless figure in a line that is being marketed as scientifically accurate. LoRusso stated that his consultants told him larger therizinosaurs would have been featherless. It's not LoRusso's fault that he somehow was able to sculpt a bald maniraptoran in the year 2013. Somebody who did not know what they were talking about and claiming to be an expert in paleoart just because they work in the related field of paleontology told him to do it, and he very reasonably believed them because they were an "expert", though obviously they had misrepresented themselves.

And there's the biggest problem and probably the answer to the question of what is going on with these strange and obvious inaccuracies. Paleoart consultants for major projects tend to be, often but not always, simply terrible. They seem not to know what they are talking about. Not only that, but second-hand reports suggest that they often simply do not care. Seriously: When asked about blatant inaccuracies creeping into paleoart-based projects like toys or books or even press releases, at least one anonymous paid paleontological consultant stated that they don't care what dinosaurs looked like in life, and so would presumably rubber-stamp any abomination that came across their desk.
Here's a prime, objective example: The Carnegie Collection Caudipteryx zoui figure. This species was first found in 1998, a complete skeleton with feather impressions. There are plenty of photos of Caudipteryx fossils that show crystal clear how the feathers attach and were ignored completely for this figure. The artist might have copied some inaccurate depiction rather than doing actual research or glancing at a fossil, and the consultant approved it because they didn't know or didn't care about the relevant details. The Carnegie Caudipteryx proves that consultants are utterly useless and often have no clue what they're talking about. Any one of us can compare the model with the fossil and show that the model is objectively wrong in major details. Look for yourself:

Caudipteryx wing fossil: note the primaries, longer than the hand, anchored along the second finger,
and lack of a clawed third finger.


Carnegie Collection Caudipteryx figure. Note the wing feathers anchored everywhere along the arm
EXCEPT on the second finger where they belong, and the incorrect number of fingers.
The wings/arms of this figure are wrong in just about every single way possible, and these are not minor details. Yet it's marketed as accurate and "paleontologist approved" in a series bearing the name of a major scientific institution!

It's not fair to ask all working paleontologists to know or care how their research into fossils translates into life appearance. Matching osteological and behavioral correlates with the structure and anatomy of living analogues could almost be considered a distinct field separate from actual paleontology. This is something paleoartists can and do think about and research constantly, but would almost never need to enter into the research when describing fossils. There's really no reason for working paleontologists to keep up to date with developments and research that go into paleoart.

The solution? Don't ask these paleontologists to consult! Just because someone is a paleontologist does not make them an expert on the life appearance of any given species of prehistoric organism. The examples cited above were, allegedly, all approved by "expert" consultants. This simply proves the consultants that are being employed are utterly failing at their job. I hate to say it, but there are legions of paleoartists and other dinosaur fans online who jump at the chance to criticize and nitpick and otherwise consult on these things for free. It's just that by the time the product is released, it's too late to do anything about inaccuracies. If companies that use paleoart would simply post concept art beforehand on, say, Facebook, they could probably get much better advice for free. Or, preferably, they could employ actual paleoartists as experts, hopefully artists who specialize in researching the life appearance of a given subject group of organisms.

Darren Naish, Mark Witton, and John Conway recently published an article on the (shameful) state of  paleoart as used in professional and commercial contexts. Companies like Safari Ltd. would do well to listen to their advice.

Thursday, August 28, 2014

Beasts of Antiquity


So, it looks like my new book, Beasts of Antiquity: Stem-Birds In the Solnhofen Limestone (Pan Aves 2014), is now available for preorder! Well, the ebook version anyway, but that's not a bad thing (see below).

Beasts of Antiquity started life as "Age of Dragons", an idea to do a dinosaur book without really talking about "dinosaurs" (inspired partly by this post). The idea was to focus on all members of the avian stem group (and talking about the historical taxon name Dracones, hence the title), not just dinosaurs, each from a different continent or formation in different books in the series. The first was going to be focused on the stem-birds of North America and would feature many of the recent illustrations on my Web site, plus obviously a lot more. Suffice it to say this is a little ambitious for a summer project, so I decided to try releasing the whole thing piecemeal in short installments based on formation first. As I recently teased on social media, this particular concept would focus on several short, stand-alone ebooks that would later be combined with new material to form a single, print volume.

Wednesday, July 16, 2014

People Think Feathered Dinosaurs Don't Look Scary. They're Right.

This short article on io9 pretty well encapsulates an area of frustration for artists and scientists in the age of feathered theropods.
Ooh, I'm shakin' in my boots.
Photo by Simon Rumble, licensed.
The implication is, right from the title, that it's common knowledge most depictions of feathered T. rex are not cool. Feathered theropods are widely derided by the public because feathers make these scary reptilian monsters less scary. In a recent Facebook discussion, I took one of those "short pelt raptor" images to task for inaccuracy (you know, the kind that pays lip service to the idea of feathered theropods, but with the minimum possible change to the classic silhouette, with a cat-like short pelt rather than a bird-like poof of feathers engulfing the body). In my reply I kind of hypothesized that there's an evolutionary psychology* reason for our aversion to feathered theropods and our cat-like concessions to the idea.

As Andrea Cau has pointed out, paleoartists (myself included), consciously or not, often employ all kinds of subtle tricks to make feathered theropods look "cool". Leaving the face scaly and reptilian is a popular trick; his body might say "Big Bird", but his face tells you he means business. Face fully feathered? Introduce an eagle-like lowered "brow" or some kind of eyebrow analogue so his facial expression can look "mean". Make sure his mouth is open or he's prominently displaying his other weapons in a ninja-like fighting stance. And be sure if you make him colorful, use high contrast, red and black if possible, and light it so his face is in shadow--that way you know he's thinking evil thoughts. This might also allow you to add eye shine making the eyes look like demonic embers! (check back to the io9 article and see how many of these points that T. rex hits).


In the comments to the io9 article, there were the predictable bouts of resistance to the idea that T. rex could have had feathers at all. "It was too large! Large mammals don't have so much fur in hot climates!" The problem with comparisons to large mammals is that feathers are very different in structure from fur, and have very different insulating properties. Fur is mainly used to keep an animal warm, but thanks to the fact that feathers grown in adjustable, planar layers, and are better at trapping and regulating air flow, many large birds use their feathers to very effectively keep themselves cool by circulation while blocking the skin from absorbing direct sun. It may actually have been disadvantageous for a large animal to lose its feathers, especially if it lived in a hot sunny climate. The fully-feathered Yutyrannus was not significantly smaller than any but the largest T. rex. Most T. rex specimens fell short of the 6.8 tons estimated for the most gargantuan known adults like Sue, that is certainly not the species average size!


But, there was one comment that played right into my ego-psych hypothesis. The commenter basically stated that we know juvenile T. rex had feathers, but there's no reason to think adults kept them. Except even that premise is wrong. 
There is in fact zero direct evidence to support the hypothesis that T. rex juveniles had feathers, let alone that they had them and then lost them. It's simply easier for people to assume that a baby animal, which is supposed to be cute, had feathers, which we psychologically associate with cute animals. 

Are one of these things is not as scary as the other?
Illustrations by M. Martyniuk, all rights reserved.

It is actually less of a stretch (i.e. more parsimonious) to hypothesize that based on its phylogenetic bracket, T. rex had feathers and retained them throughout its life, than the hypothesis that T. rex was born with feathers, lost them because they became disadvantageous at some unspecified weight, then through some unknown developmental pathway replaced its feathers with the kind of thick, scaly skin it is usually depicted with and would need to protect itself from the sun/injury if it lacked feathers. But this convoluted thinking is easier for people to accept because T. rex is the king of all monsters, and monsters are by definition not cute.**

The sad fact is, T. rex may not have looked all that cool. I think John Conway and others have brought this up before. It, and many if not most other dinosaurs, may very well have looked really, really stupid to us. Nature doesn't care if an animal looks intimidating to a species that evolved 66 million years later in a completely different environmental context alongside a vastly different set of predators. Our brains are programmed to find mammalian and reptilian predators scary at least in part* because we evolved alongside these and our survival depended on it. We had no such pressure for most kinds of birds***, and maybe coincidentally, we find very few kinds of birds the least bit intimidating. We have to be told/shown that a cassowary is even capable of being dangerous, and people still constantly trot this out as a surprising fact, despite the fact that it has very few physical differences from a Velociraptor, other than being much larger! 


So, if your average Joe met a non-avialan theropod in real life, the reaction might be less like any of the raptor scenes in the original Jurassic Park and more like Newman vs. the cute, colorful, silly, hopping (read: bird-like) dilophosaur - bemusement leading to injury.

* I know evo psych is mostly made up of untestable just-so-storys. But it's still fun to think about.


** That's sarcasm. Tyrannosaurs were not monsters, they were plain old regular animals. A lesson people forget from the original Jurassic Park (probably because they're not actually depicted hat way in the movie, despite the fact that the characters talk about it).


***Raptors seem to be the exception. Probably because they preyed on early humans, and maybe also because of their mean-looking "eyebrows"?


Sunday, September 1, 2013

You're Doing It Wrong : Dino Foot Scales

Above: Our subject matter.
It's often said by those who support a strict phylogenetics-based system of naming life that it's only by restricting well-known names from neontology (the study of modern organisms) to crown groups can we avoid making unjustified assumptions about members of stem-groups.

These kinds of unjustified assumptions have been rampant in the history of studying stem-birds. Archaeopteryx has traditionally been depicted, incorrectly, with a reversed hallux, and occasionally even with beak-like structures, simply because it's a "bird", and those are features all birds have. Except Archaeopteryx is not a true "bird", it's a stem-bird, more closely related to birds than to any other living animal group, but not a member of the group that includes all modern birds. It's fair to assume that an extinct member of the duck lineage, like Vegavis, had a bill, but that's not necessarily so for, say, Patagopteryx, despite the fact that it is usually referred to as a "bird".

Modern bird feet, by Philip Henry Gosse, 1849, public domain. Note overlapping scutes on
the top surfaces, and pebbly, polygonal reticulae on the bottom surfaces.

Most paleoartists have absorbed these kinds of warnings, and do a good job of avoiding obvious errors based on typology, the assumption that all species in a certain "type" share "key characteristics." But there are some typological memes in the bird lineage that are more pernicious, possibly because their actual evolution is something most artists don't think about very much.

Take, for example, the bird-like scutes that are almost universally illustrated covering the tarsus (upper foot/lower hind limb) of dinosaurs. Is there any evidence that these were actually present in any given group of non-theropod stem birds? Well... no. Not that I'm aware of (if you know differently, please comment!).

Sinosauropteryx prima with tarsal scutes.
Image by Matt Martyniuk,  licensed.
I'm not sure when this meme began, and if it's related to the Dinosaur Renaissance when the link between birds and dinosaurs was re-established. Looking at some Charles Knight paintings, such as his famous "Leaping Lealaps", it appears that the feet of his theropods were scaled based on modern lizards (more on the differences between lizard scales and other types of "scales" below). Bakker's influential early restoration of Deinonychus does not include any obvious scutes on the feet or tarsus. Mark Hallet, on the other hand, did include what look like oblong bird-like scutes on his theropods. At any rate, it's hard to deny that "bird feet" are typical of almost all modern reconstructions of dinosaurs, including my own, and are not limited to theropods. Bird-feet are often restored on ornithischians and even pterosaurs.

Of course, like many paleo-memes that developed during the 1980s, the main idea seems to be using this as a flourish to make otherwise scaly dinosaurs seem more bird-like. And thanks to skin impressions, we know that many dinosaurs had scales, right?

Tuesday, June 4, 2013

You're Doing It Wrong: CGI Feathered Dinosaurs

YIKES.
Promotional still from When Dinosaur Roamed America,
Discovery Channel 2001
CGI dinosaurs have come a long way since Jurassic Park. Unfortunately, due to the discovery that these animals were far more bird-like than reptile-like, that direction is straight down a seemingly bottomless pit. For many CGI artists and animators, the key concept that is presenting a very steep learning curve is the idea that these animals need to be restored as feathered dinosaurs, not "dinosaurs with feathers." It looks like many people modeling feathered dinosaurs start out by rendering a featherless dinosaur and then using various modeling or rendering tricks to add the feathers. As you'll see below, this never, ever works.

Saturday, May 11, 2013

The Validity of Lambeosaurus - Anybody Know A Good Lawyer?

Reconstruction of Didanodon altidens specimen ROM 794 (aka Lambeosaurus lambei,
aka Procheneosaurus praeceps) by Matt Martyniuk, all rights reserved.
I've talked a lot on this blog about my personal justifications for using "old fashioned" names for many groups or species of stem-birds. In many cases, names which were in common use during the 19th and early 20th centuries were replaced later by one or two influential scientists for reasons which don't really hold up when you look at the codes that govern naming in biology. For example, Manospondylus gigas may currently be the correct name for the theropod we know and love as Tyrannosaurus rex, but this possibility has almost never been discussed because everybody assumes it's a nomen oblitum - a name out of use for so long that it becomes automatically invalid under the International Code of Zoological Nomenclature (ICZN). Note the word "assume"--as I've written before, most people, even working scientists, don't really know what criteria must be met to classify a name as obsolete.

The name of one very well-known dinosaur is in such a sorry state that it's like the Manosponylus / Tyrannosaurus debacle squared. The genus Lambeosaurus, a well-known hadrosaurid with a distinctive squared-off crest with a backward-pointed prong, was named twice prior getting its popular moniker, and neither of those names can be considered obsolete, since they were both coined during the 20th century.

The first name given to fossil material (in this case a jaw) now universally attributed to Lambeosaurus was Didanodon. In a 2006 review of hadrosaurs, Lund and Gates stated (without discussion) that the genus and its type species, Didanodon altidens, were nomina nuda, or "naked names" lacking the proper description necessary to establish them. But is this really the case?

Monday, December 5, 2011

Waddle, _Achillobator_, Waddle!

Above: Revised illustration of Achillobator giganticus with corrected leg proportions. Scale bar = 500 mm. By Matt Martyniuk, all rights reserved.

"I've hunted most things that can hunt you, but the way these things move..."
"Fast for a biped?"
"Cheetah speed. Fifty, sixty miles an hour if they ever got out into the open, and they're astonishing jumpers."

This quote from the original Jurassic Park film did much to cement the image of dromaeosaurids, the raptor* dinosaurs, in the public consciousness as fleet-footed hyper predators. Despite being nearly 20 years old, this portrayal has by and large remained unchanged in popular culture, with raptors often stock monsters with near-supernatural murderous abilities in everything from tongue-in-cheek xkcd comics to (I hope) tongue-in-cheek made for SyFy movies.

*Yes, I'm going to commit a cardinal sin and refer to dromies as "raptors". "Raptor" in ornithology refers to most predatory birds, even those that hunt on the ground (the Raptor Research Foundation considers Secretarybirds to be raptors). Since dromaeosaurids were both predatory and birds under any sane definition of the word, there should be no problem referring to them as an extinct group of raptors.

But were raptors really particularly fast? Bipedal running speed in digitigrade animals (that is, those that walk on their toes like birds rather than their ankles like humans) is usually roughly determined by the ratio of the lower leg bones (the tibia/tibiotarsus) to the upper foot bones (the metatarsus). The longer the upper foot is in length compared to the lower leg, the faster an animal could run. Therefore, we would expect the fastest theropod dinosaurs to be those with the longest metatarsi relative to tibiae.

A prime example of a theropod specialized for running very very quickly are the parvicursorines. This specialized group of alvarezsaurids (strange theropodan insectivores with stout, powerful arms each bearing one very large claw) has among the longest lower leg to upper leg ratio of any Mesozoic dinosaur group.  Looking at the statistics compiled by Mickey Mortimer at The Theropod Database (a phenomenal resource I turn to so often I really should just make it my browser's home page), the type specimen of Parvicursor remotus (see leg diagram here) has a femur 52.6 mm long, a tibiotarsus about 75.6 mm long, and a metatarsus 58 mm long. The functional lower leg is 113 mm long, well over twice the length of the upper leg. More importantly, the lower leg and upper foot bones were fairly close to being equal in length. This animal was clearly a speed demon.

How does this compare to raptors? If, as Jurassic Park claimed, raptors were exceptionally fast, we would expect them to have similarly long lower legs. The terrifyingly human-sized raptors in JP were a Hollywood invention, but we do know of raptor species slightly smaller and slightly larger than they were.

On the smaller side were the famous Deinonychus antirrhopus. According to TTD, the femora of one relatively complete specimen measured 248 mm, with a tibia 324 mm long, and a metatarsus 151 mm long. Again, the total lower leg length is nearly double the upper leg. But the upper foot bones were only half as long as the lower leg bones.

The "fast raptor" meme was started by John Ostrom himself, when he first described Deinonychus in 1969. This was merely speculation on his part, as the hind limb was not completely known in the first specimens. Ostrom actually changed his opinion in later papers, finding that the femur was shorter than he'd initially thought, and that the foot bones were surprisingly short compared to other dinosaurs. Not only was Deinonychus not particularly fast, it probably could not have been nearly as fast as most other small theropods, including modern flightless birds, let alone cheetahs.

Another very popular type of raptors are advanced giant dromaeosaurines (Utahraptor and Achillobator). I recently found myself revising an older drawing of an Achillobator giganticus, which were, as mentioned above, only slightly larger than the Jurassic Park raptors. Many young dinosaur fans are very attached to these species in part because they're much larger than most other raptors, and because they had a slightly anthropomorphized novel written about them by Bob Bakker shortly after JP was released (Raptor Red). As a result, these big birds have a cachet in the collective consciousness similar to the generally more famous Deinonychus and Velociraptor--that of super-fast, agile and intelligent predators.

However, when finishing up my revised drawing, I had to double check the proportions several times to make sure I wasn't screwing it up. To my amazement, the legs, particularly the lower legs and upper foot bones, looked almost laughably short. Again according to TTD, the femur of A. giganticus measures 505 mm long, the tibia 490 mm long, and the metatarsus a paltry 234 mm long--less than half the length of the tibia. Not only is the metatarsus much, much shorter than the tibia, the entire lower leg in only marginally longer than the femur! The first thing that struck me wen looking at my own reconstruction was that this looked like the dromaeosaurid equivalent of Majungasaurus, those abilisaurids with the ludicrously short legs (which, coincidentally like Achillobator, have been suggested to be made up of chimeric specimens). It is also reminiscint of another stout-legged dromaeosaurid species, Balaur bondoc. While Balaur have been suggested to be possibly herbivorous due to these strange proportions, partial jaws and some teeth of Achillobator confirm that they were carnivores. But with legs like those, it's hard to imagine these creatures behaved the way the public imagines raptors to have done, chasing down fast moving prey. Frankly, it's hard to imagine Achillobator doing much beyond waddling across Nemegtian lake shores hunting turtles in epic slow-motion chases.

For the record, no described specimen of Utahraptor preserves both a femur, a tibia, and a metatarsus, so it's impossible to say whether or not they had the same squat proportions (unless somebody has some more detailed information on the numerous undescribed specimens in the BYU collections). For now, it would be safe to assume that they, too, would have been a laughing stock if they were caught trying to run.

Ok, but why would predatory animals have such stubby legs? There is a lot of evidence that dromaeosaurids were specialized for hunting big game, often animals larger than themselves. Deinonychus are infamous for their association with large ornithopods Tenontosaurus tilletti, and while evidence suggests they mainly targeted juveniles (Forster 1984), these were still much larger in terms of weight than even adult Deinonychus. Velociraptor are known to have grappled with the larger Protoceratops, and even a rumored specimen of a Microraptor apparently preserves evidence that they tackled prey larger than themselves. The short legs, especially the short foot bones, seem to be linked with the function of the large sickle-claw, making lack of speed a trade-off for improved ability to grapple and kill large game. Dinosaurs like Tenontosaurus and Protoceratops probably weren't particularly fast-moving themselves, making this sacrifice in speed worthwhile for the chance to down a massive animal that could provide a whole lot of food.

In the end, while the raptor chase scenes in Jurassic Park remain some of the most exciting parts of the movie, they require a significant amount of disbelief to be suspended; after all, it would be more realistic but slightly less suspenseful if Laura Dern had been able to evade the raptors in the power bunker by simply breaking into a light jog.

Saturday, November 19, 2011

Who's That Birdie?

Because I initially got the inspiration for tomorrow's big post while working on the new restoration above, I thought I'd post it alone first as a teaser. First to correctly guess the species gets a shout-out!

Friday, September 16, 2011

Feathers ARE Color

A lot of my posts lately have been dedicated to color in prehistoric feathers (primer here). As a  paleontographer, it's hard not to get excited about finding new ways to more accurately and naturally depict long-gone animals, and I know a lot of you reading this feel the same way. It can also be frustrating knowing the basic color palate we're dealing with, but having specific data from only a handful of species to draw inspiration from. I've already seen, not surprisingly, a few illustrations of Microraptor, Xiaotingia, etc. that basically mimic Anchiornis down to the spangles. We're so conditioned to follow phylogenetic bracketing that it's tempting to use what little info we have, and extrapolate it to close (and even not so close) relatives. This can apply to larger feather patterns as well; as I mentioned in this post, it's fine to extrapolate Microraptor-style feathering to Velociraptor, but it's not the ONLY way to do it, nor is it even necessarily the most plausible for a creature of such different size and ecosystem, as many online critics of Dinosaur Revolution would have you believe ;)

With that in mind, I want to start with a disclaimer: this kind of info only gets you so far. I'm not setting out to write the inerrant Bible of paleoart in these types of posts. Yes, all the evidence we have of dromaeosaurs shows full, lush feathering equivalent to small modern birds. But then again, we're dealing with small prehistoric birds here. Yes, we can interpret feather coloration and use inferences from modern birds and biochemistry to say what colors are likely and which are unlikely; but we can't always identify structural color in fossils, and we have yet to identify carotenoids, and many small dinosaurs we think of as "carnivorous" might well have trended more toward omnivory, insectivory, etc., or other unforeseeable pathways to those tasty, tasty bright yellow pigments.

Ok, preamble out of the way, the point of this post is to provide a general way I've used, and others can use, to try to make somewhat educated guesses about coloration in prehistoric birds which have not yet been analyzed for color pattern.

A few people pointed out to me when this recent paper by Wogelius et al. came out, in which the research team was able to identify color patterns in some Mesozoic birds using chemical markers rather than direct observation of melanosomes, that their reconstruction of Confuciusornis based on these findings was pretty similar to the restoration I'd done a while earlier.


Above: Restoration of Confuciusornis by Richard Hartley, from the press release. Below: My own earlier restoration of C. sanctus.


The two are pretty similar in the broad pattern: dark head, body, and coverts, white or light-colored wings with more black on the secondaries than the primaries. Now, so far this is only one data point, so I don't want to draw too many conclusions. But I was not simply guessing when I restored C. sanctus that way back in 2009.

The trick is to understand what you're looking at when you see a fossil feather. These are often referred to as 'impressions', but often the impressions are only part of the story, or even completely absent from the fossil. The breakthrough that led Vinther , Prum and others to figure out how to suss out feather color, was in realizing what fossil feathers are made of.

As Prum summarized on the Skeptics Guide to the Universe podcast a few years back, traditional wisdom held that the dark, 'carbonized' looking fossil feathers were the result of bacteria. Now, some old-school feather impressions, like those from Solnhoffen and the Santana formation, do contain nice, deep, actual impressions. These look very different from the stuff you find in the Jehol (compare the fossil feathers of the Berlin Archaeopteryx with the holotype of Microraptor gui). But most fossil feather,s including the famous single-feather holotype of Archaeopteryx and most Jehol stuff, are dark stains in the rock. Under the microscope, these looked to early researchers to be made up of fossil bacteria which had eaten away the feather keratin during decomposition.


Above: Photograph of an unsubscribed Anchiornis specimen by Robert Clark, from National Geographic, showing clear color patterns matching those predicted by Vinther et. al.

What Prum, Vinther, etc. showed in recent years is that this is flat-out wrong. Those granules are not bacteria--they're melanin! When you look at a fossil feather, most of the time, you're looking directly at the color pattern of the feather itself, the keratin and everything else having long since disappeared. This is especially apparent in very well-preserved fossils; for example, the beautifully preserved new Anchiornis specimen above is essentially proof of Vinther's hypothesis, which had previously been based on more obscured differences in shade. This is where my method of eyeballing it falls flat--I'd never have gotten the correct pattern from the specimen Vinther was looking at without really close physical examination. You need really nice specimens for it to conceivably work, or you have to Dave-Peters the heck out of low-res images trying to spot differences in contrast on the feathers.

Luckily, Confuciusornis was a safe bet, because so many specimens are known, and you can start to see patterns emerge. Many of the best specimens tend to have a very dark halo of feathers around the body and arms, with the wing feathers very faint, even sometimes difficult to see at all. Knowing that dark feathers means dense melanin = dark coloration, and light color = lack of melanin = light color, it was easy to come up with a good guesstimate of the life coloration. This was first inspired by Longrich's work on Sinosauropteryx, showing that the apparent bands in the tail were due to color patterning, which was later supported by published studies.

Obviously this is not a foolproof method. But it's a good place to start for artists who may want to add a little evidence-based thinking to their reconstructions, even if the evidence itself is wide open to interpretation. At the very least, if a good specimen has obvious areas of light and dark, I'd personally restore that pattern in a life illustration. It may end up being wrong, but it's better than pure speculation.


Monday, May 30, 2011

Know When To Fold 'Em


Above: Maximum wrist folding for the theropods studied by Sullivan et al. 2010. Not to scale.


(Cross-posted from Art Evolved)

To continue talking about aspects of maniraptoran anatomy that can be a bit vaguely defined in the minds of paleoartists, I'm going to write a bit on the issue of wrist folding. As most of you will know, a major characteristic of maniraptorans is the semi-lunate carpal, the half-moon shaped bone in the wrist that allows the blade of the hand (metacarpal 3) to fold backward toward the forearm (ulna). While this is common knowledge among paleo buffs and artists, what seems to be less understood is exactly how tightly the hand (and in aviremigians, the wing) could actually fold up. I myself have never been too clear on the issue, and there don't seem to be many papers addressing this. But in the last few years, a few papers have come along that can help shed light on the subject. The first was Senter 2006, which studied the full range of motion in the forelimbs of two dromaeosaurs, Deinonychus and Bambiraptor. The second was Sullivan et al. 2010, which examined the range of motion in the wrist of several species representing each major group of non-avialan maniraptorans.

Both papers, however, present geometric data that can come across as a bit inaccessible for your average artist, so I'm going to try to break down their conclusions for those of us who are more visual thinkers. The Sullivan paper, in particular, discusses the degree to which the wrist could fold, but doesn't necessarily provide diagrams or even final angle between the metacarpals and ulna for each species that could be used as a simple reference. I've done my best to translate their findings into the image at the top of this post, using modified skeletal diagrams by Scott Hartman and Jaime Headden.


Above: Anatomy of a maximally folded wing of the Wild Turkey Meleagris gallopavo, modified from Sullivan et al. 2010
The degree of wrist folding is controlled by two wrist bones. The cuneiform, on the inside where the wrist meets the bottom of the distal ulna, provides an inner limit. The cuneiform blocks the hand from actually touching the ulna. The radiale, on the outside of the fold, forms the surface which the wrist cannot fold beyond. This is basically a little process anchored to the tip of the radius where the top part of the hand articulates. The hand can obviously not fold beyond the angle of the radiale, or the animal would dislocate its wrist. Therefore, the angle the articular surface of the radiale forms with the ulna is used as the key factor in determining maximum wrist folding by Sullivan et al. Again, see my interpretation at the top for how their results likely translate into life position.
The results show that in almost all maniraptorans, the wrist could not be folded to the same degree as modern birds (for comparison, see the photo of the turkey wing above, which is at its own maximum folding point). Note that in actual, functional angle of folding in the turkey is 57 degrees between MCII (where the feathers attach) and the ulna. To see how this translates into a live animal, here's a photo of wild turkeys nicely showing the way the feathers fold (photo by D. Gordon E. Robertson, from Wikipedia, licensed):
The wrist is located about where the coverts form the point of a triangle, following the line formed by the border of the the brown secondary (ulna) feathers and white banded primary (metacarpus) feathers. Note that with the wrist folded at a 57 degree interior angle, the feathers (especially the secondaries, which help cover the primaries when folded) are basically stacked one on top of the other with little to no fanning out at the tips. This is because the feathers also have some ability to move at their bases, and can themselves fold relative to their anchor bones through muscle and ligament action.

Looking at the aviremigians in the diagram up top, it is apparent that their wrists could not fold tightly enough to fold the wing feathers to the same degree as a modern turkey. Small deinonychosaurs like Sinovenator and Bambiraptor could achieve close to a 100 degree angle (see image of Bambiraptor wing folding above, from Senter 2006), but larger ones like Deinonychus seem to have lost some of that folding ability, presumably for increased use of the forelimbs in predation. Indeed, if Deinonychus retained long remiges, they would hardly have been able to fold at all, and would have been permanently fanned out (not that this would have gotten in the way of grabbing prey, as Senter pointed out). This lack of ability to tightly fold the wrists may have posed a significant problem for those species with very long remiges, like Microraptor gui. Dave Hone, who was a co-author of the Sullivan paper, discussed alternative ways they could have kept their remiges free of the ground at his blog last year.

In pygostylians, the degree of wrist folding began to approach that found in modern birds. Eoconfuciusornis, for example, could fold its wing to about the same degree as a turkey. Where it gets weird is in the oviraptorosaurs. As I mentioned in my post on the Ashdown maniraptoran, oviraptorosaurs (at least the small basal ones like Caudipteryx) seem to have been capable of folding their wings far beyond what is possible for even many modern birds. It's unclear why this is so, especially as the remiges of Caudipteryx, while clearly for display, are not exactly very long compared to the body. Certainly its wings were much smaller than those of paravians, which would have presumably had more need to fold them up. I've seen this mentioned as possible evidence in support of the hypothesis that oviraptorosaurs are in fact avialans, and that the extreme folding of the wrist was inherited from flying ancestors, though I can't think of where. Sullivan et al. do note that more than folding up the remiges to keep them safe from wear and tear, wing folding is an important part of the avian flight stroke, and it makes sense that it would have become more developed in flying forms.

Anyway, we've only got a handful of specimens that have been specifically studied in regards to the degree of wrist folding, and there may well be exceptions in each maniraptoran group, where certain lineages independently evolved a greater or lesser degree of wrist folding from their ancestors as seems to have happened in therizinosaurs, where the derived Alxasaurus can fold its wrist more than the basal Falcarius, and deinonychosaurs, where the relatively derived Deinonychus can fold its wrist less than the more basal Bambiraptor. So this guide shouldn't be considered as a set of hard and fast rules, but rather a starting point for artists who want to make their restorations as plausible as possible.

Finally, a few days ago I posted a teaser for this post challenging people to determine what aspect of the above Deinonychus illustration was incorrect. By now it should be clear that the wrist is folded too far back. Appropriately enough, the first one to nail it was the artist, Nobu Tamura, himself! Commenter A.G. came close, speculating that it was due to the orientation of the glenoid, but that has more to do with the range of motion of the upper arm and how far it could extend into a bird-like flapping position, rather than the way the wing folds up. Good job guys!

References
* Senter, P. (2006). "Comparison of Forelimb Function Between Deinonychus And Bambiraptor (Theropoda: Dromaeosauridae)". Journal of Vertebrate Paleontology, 26(4): 897–906.
* Sullivan, C., Hone, D.W.E., Xu, X. and Zhang, F. (2010). "The asymmetry of the carpal joint and the evolution of wing folding in maniraptoran theropod dinosaurs." Proceedings of the Royal Society B, 277(1690): 2027–2033.