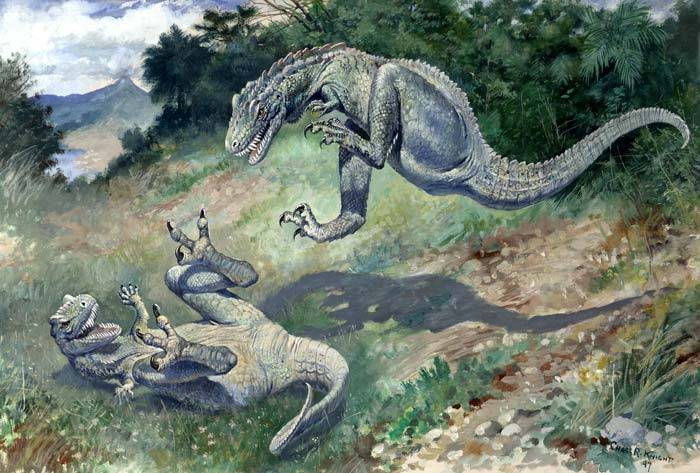Showing posts with label biology. Show all posts

Wednesday, April 12, 2017

You're Doing It Wrong: Pteranodon Bills

Your bill's looking a little puny, there, buddy.
(Painting by Heinrich Harder, 1912, public domain).
Everybody knows Pteranodon. Quick, stop to imagine it! It's easy, because it's the most often-illustrated and well known pterosaur to the general public (though today's marketing departments often call it a pterodactyl, following it's original, century-out-of-date classification).

But hold on. That image you have in your head right now, of a big pterosaur with a long crest and a mid-length pointy beak? That's likely wrong, and may be just as much a hybrid as those Flintstones-style creatures with pteranodont crests and Rhamphorhynchus tails.

How do we know? Let's talk about Dawndraco.

Saturday, February 21, 2015

The Evolving View of Stegosaurus

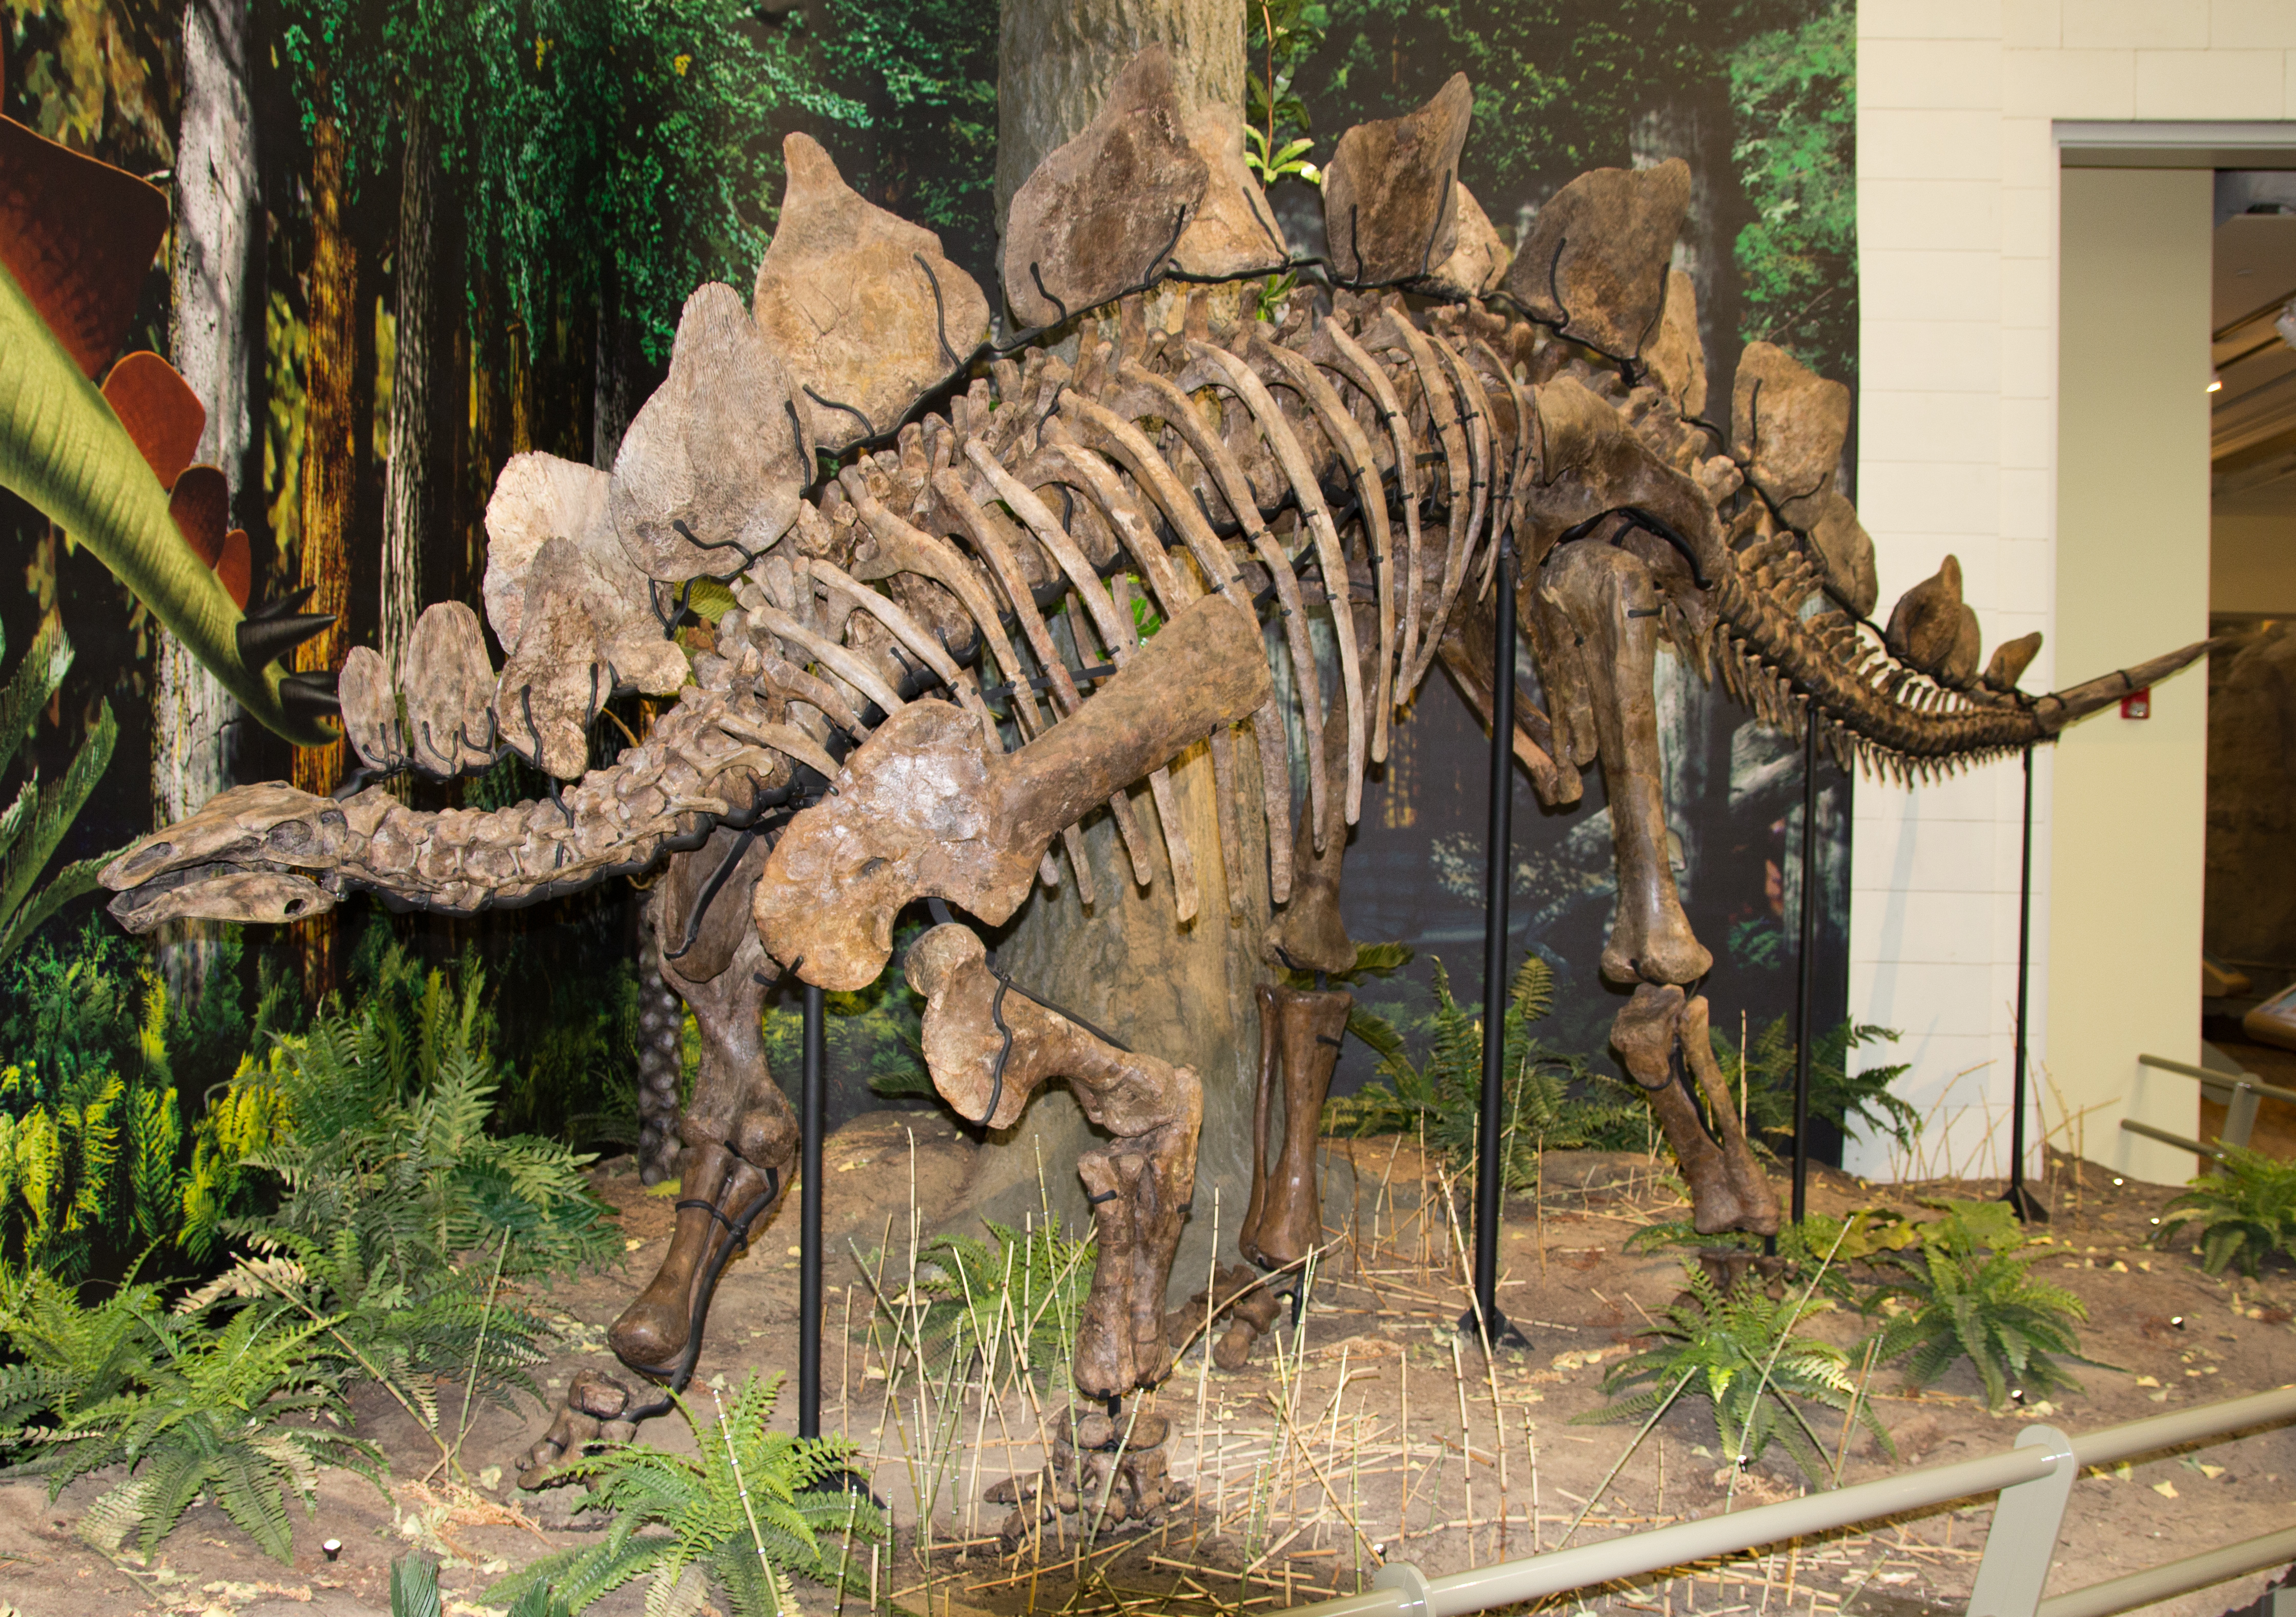
Mounted skeleton of Stegosaurus ungulatus at the Carnegie Museum. The tail, plate, and spike arrangement have been updated in this mount to reflect current thinking following the study by Carpenter (1998). Photo by Perry Quan, CC-By-SA 2.0.
Seeing as how I've been working on restorations of two different stegosaur species this month, I thought I'd write up a quick review of the most famous aspect of these iconic dinosaurs: Their big, triangular plates. For a complete overview of the history and interpretation of Stegosaurus, be sure to see Ken Carpenter's 1998 paper.

Interpretation of the life appearance of stegosaurs has changed several times since they were discovered by O.C. Marsh in 1877. The first stegosaur fossil (belonging to the species S. armatus) were found near the town of Morrison, Colorado, but the specimen was disarticulated and only a few of the plates were preserved. Initially, Marsh thought that these plates played flat along the animal's back, forming a sort of turtle-like shell, or like the tiles on a roof (hence the name Stegosaurus, which means "roofed lizard"). Marsh also initially believed that stegosaurs were aquatic, due to this turtle-like appearance, but also that they would have walked on two legs on land.

Sunday, June 15, 2014

What Does T. rex Say?

"Hissssssssssssssssss!"
T. rex holotype specimen. Photo by Scott Robert Anseimo, CC BY-SA 3.0.
It's an iconic scene in every dinosaur movie: the huge, conquering carnivorous theropod rears back and lets out a terrifying bellow. Sound effects artists spend huge amounts of time sampling vocalizations from various animals to create just the right mix to create an unfamiliar, otherworldly roar. And, of course, everybody knows that pterodactyls let out harsh, echoing, prehistoric sounding screeches.

But how close to reality are these sounds? Do we have any ways of using science to figure out what dinosaurs and other stem-birds may have sounded like? Do we have evidence that they made sounds at all?

Sunday, September 8, 2013

Iridescence in Simple Feathers - The Case of the Blue Troodon

Iridescent feathers in troodontids - possible? Image by Matt Martyniuk, all rights reserved.
(Supreme dino fans may recognize the pose even from this small clip...)
I've written a lot about the various ways feathers get their color in order to create some rough guidelines for paleoartists restoring feathered stem-birds. I recently had a quick discussion over at DeviantArt with one of the best currently-working paleoartists around, Emily Willoughby, over the plausibility of a blue Troodon. Note that it has a few other anatomical issues that make it somewhat less than a fully accurate rendition, but is the coloration one of them? I wasn't sure, so I did a little extra digging to find out. As usual, this research is cursory and I welcome any additional input on research or details I may have overlooked.

Sunday, September 1, 2013

You're Doing It Wrong : Dino Foot Scales

Above: Our subject matter.
It's often said by those who support a strict phylogenetics-based system of naming life that it's only by restricting well-known names from neontology (the study of modern organisms) to crown groups can we avoid making unjustified assumptions about members of stem-groups.

These kinds of unjustified assumptions have been rampant in the history of studying stem-birds. Archaeopteryx has traditionally been depicted, incorrectly, with a reversed hallux, and occasionally even with beak-like structures, simply because it's a "bird", and those are features all birds have. Except Archaeopteryx is not a true "bird", it's a stem-bird, more closely related to birds than to any other living animal group, but not a member of the group that includes all modern birds. It's fair to assume that an extinct member of the duck lineage, like Vegavis, had a bill, but that's not necessarily so for, say, Patagopteryx, despite the fact that it is usually referred to as a "bird".

Modern bird feet, by Philip Henry Gosse, 1849, public domain. Note overlapping scutes on
the top surfaces, and pebbly, polygonal reticulae on the bottom surfaces.

Most paleoartists have absorbed these kinds of warnings, and do a good job of avoiding obvious errors based on typology, the assumption that all species in a certain "type" share "key characteristics." But there are some typological memes in the bird lineage that are more pernicious, possibly because their actual evolution is something most artists don't think about very much.

Take, for example, the bird-like scutes that are almost universally illustrated covering the tarsus (upper foot/lower hind limb) of dinosaurs. Is there any evidence that these were actually present in any given group of non-theropod stem birds? Well... no. Not that I'm aware of (if you know differently, please comment!).

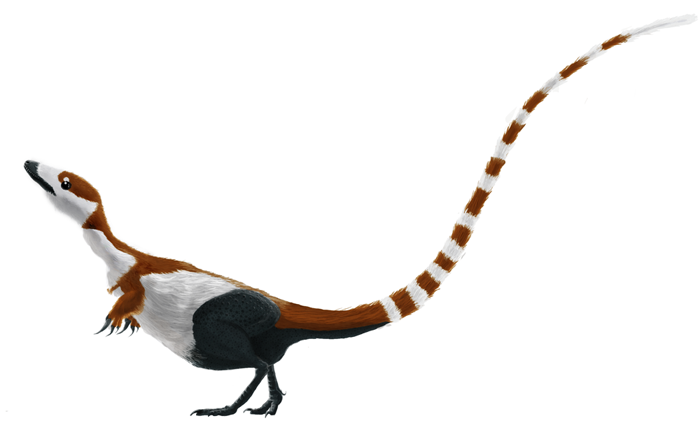
Sinosauropteryx prima with tarsal scutes.
Image by Matt Martyniuk,  licensed.
I'm not sure when this meme began, and if it's related to the Dinosaur Renaissance when the link between birds and dinosaurs was re-established. Looking at some Charles Knight paintings, such as his famous "Leaping Lealaps", it appears that the feet of his theropods were scaled based on modern lizards (more on the differences between lizard scales and other types of "scales" below). Bakker's influential early restoration of Deinonychus does not include any obvious scutes on the feet or tarsus. Mark Hallet, on the other hand, did include what look like oblong bird-like scutes on his theropods. At any rate, it's hard to deny that "bird feet" are typical of almost all modern reconstructions of dinosaurs, including my own, and are not limited to theropods. Bird-feet are often restored on ornithischians and even pterosaurs.

Of course, like many paleo-memes that developed during the 1980s, the main idea seems to be using this as a flourish to make otherwise scaly dinosaurs seem more bird-like. And thanks to skin impressions, we know that many dinosaurs had scales, right?

Saturday, April 20, 2013

Supporting the Dinosaur/Bird Link in the Era of the MANIAC

I'm posting this more as an open question than a statement of my own opinion, so comments appreciated!

A new paper out in Paleobiology by Verracchio et al. describes the porosity of Troodon formosus eggs and uses the data as evidence to support the hypothesis that troodontids brooded their eggs, like modern birds and other known maniraptorans, rather than burying them, like crocodilians and some other modern birds. In and of itself, this conclusion is interesting in that it pretty much solidifies nest brooding (as opposed to burial) as the ancestral trait for modern birds, and for maniraptorans (or at least chuniaoans*) in general.

Study coauthor Darla Zelenitsky with Troodon formosus nest. Photo by Jay Im, University of Calgary.
I hate to admit it, but my first thought when reading the headline of this news article from PhysOrg was that, yeah, we all assumed that anyway. The unspoken "rule of cool" is that science tends to be more exciting when we find evidence that contradicts previously well-supported hypotheses, rather than confirming hypotheses we all took for granted. Sure, finding the Higgs-Boson was exciting, but not nearly as exciting as not finding it, which could have led to new physics. I assumed, and I'm sure many others did as well, that troodontids brooded their eggs, based on the reasonably secure hypothesis that oviraptorids (which are known to have done so) are more basal. This behavior in troodontids was even depicted nicely in 2011's Dinosaur Revolution. So score another one for phylogenetic bracketing!

(Of course, this is not to imply that all chuniaoans must have brooded their eggs. It's entirely possible that reversals to burial nesting occurred, as with modern megapodes, and this seems especially likely for very large species like some dromaeosaurines. But the odds that any given chuniaoan would not be a brooder are low.)
Arctic troodontids, anatomy based on Troodon formosus.
Matt Martyniuk, all rights reserved.
Aside from all that, the assertion in the PhysOrg headline struck me as particularly meaningless. How could a study of troodontid brooding lend support to the dinosaur/bird hypothesis? This statement would have been accurate a decade ago, but not today. The reason is the moving goalposts of the dinosaur/bird opposition.

Wednesday, April 10, 2013

What's A Monoclonius?


Hypothetical restoration of an adult Monoclonius crassus,
by Matt Martyniuk. All rights reserved.

Monoclonius crassus is an iconic ceratopsian, a fixture of many 1970s era dinosaur books, which owes its status almost completely to another species. 

I grew up with depictions of Monoclonius in media like Phil Tippet's short film Prehistoric Beast and toys like the DinoRiders figure. Like most representations of Monoclonius in popular culture, these were based on specimens now classified as Centrosaurus apertus (though, actually, that DinoRider looks like it has a genuinely Monoclonius-type frill, long, straight, and unadorned). 

Originally known only from teeth and a fragmentary frill and nasal horn, the Monoclonius was one of the first ceratopsians known to science, found by E.D. Cope in 1876 and named for its configuration of tooth roots ("single sprout" as opposed to the "double sprout" of Diclonius, now known to pertain to a hadrosaur). 

Like many of Cope's species, Monoclonius was not recognized for what it really was (a "horned dinosaur") until more complete remains from other ceratopsians likeTriceratops were found by Cope's rival O.C. Marsh. Monoclonius itself remaned enigmatic for many years, though the idea of a Triceratops-like ceratopsian with a single large nasal horn was used by Charles R. Knight in his famous painting of Cope's other dubious ceratopsian, Agathaumas. Knight also incorporated spiny dermal armor associated with some supposed Monoclonius remains, though at least some of this material was later shown to belong to ankylosaurs and pachycephalosaurs.

Monoclonius became iconic when complete skeletons of ceratopsians were found in the Judith River/Dinosaur Park Formation of Montana/Alberta. In the early 1900s, C.H. Sternberg (who had co-discovered the orgiinal Monoclonius fossils with Cope) established that complete specimens classified by Lawrence Lambe as Centrosaurus apertus (and some of which were considered to be Monoclonius and which had already been used to form a picture of that animal) were a distinct species. After this, the genus Monoclonius was dismantled, with former specimens re-assigned to either new or recently established centrosaurine genera.

Matters were complicated by the discovery of the drastic changes centrosaurines went through as they grew, and today the distinctive Monoclonius specimens are generally considered juvenile centrosaurines. Zach Miller has done an awesome rendering of a centrosaurine growth series showing where a traditional "Monoclonius" specimen fits into the sequence. 
Skull of the subadult Monoclonius lowei. Note the three prominent projections at the rear of the
 parietal frill. Incipient styracosaur-like spikes?

However, known specimens of Monoclonius aren't a perfect match for juveniles of the contemporary Einiosaurus, as Miller notes. The long, generally flattened frill with larger incipient spikes at the first three positions of the the parietal (Ryan 2006) are reminiscant of Styracosaurus and Einiosaurus, all of about the same geological age. The large size of a specimen sometimes referred to the distinct species Monoclonius lowei compares with some pachyrhinosaurs like the contemporary Achelousaurus, and while these do begin life with a small nasal horn that later develops into a boss, and though it isn't backward-cureved, such drastic changes during ontogony are known in other ceratopsians. It may be that Monoclonius is a juvenile form of (and therefore a senior synonym of) one of these centrosaurines, or it may be a valid species similar to both, possibly a transitional form between centrosaurin-type centrosaurs and pachyrhinosaurs. Ironically, though long mixed up with that genus, Monoclonius doesn't seem to be as great a match for Centrosaurus itself.

In my restoration of a hypothetical, mature Monoclonius (above), I made it generally styracosaur-like, though with more einiosaur-like parietal spikes, and these could alternately be seen as styracosaur parietal spikes which are not yet fully grown. In this way I've tried to hedge my bets: this Monoclonius could either be a mature, intermediate stage between styracosaurs and einiosaurs, or simply an immature but very large styracosaur. 

The nasal horn is restored as styracosaur-like as well, a conservative growth trajectory for the shorter, recurved nose horn seen in subadult specimens of M. crassus and M. lowei. However, it's entirely possible that as the nasal horn grew, it swept forward into the hook-like horn of Einiosaurus or even flattened and thickened into the nasal boss seen in Achelousaurus. Both of those pachyrhinosaurs have long parietal spikes like Monoclonius seems to have had, though both only had a single pair jutting from the back of the frill, while Monoclonius seems to have been developing at least three. Though, again, it's possible the transformation was more extreme than I'm assuming for my illustration, and that these incipient parietal horns were resorbed during growth like the epiparietals of chasmosaurines (e.g. Triceratops).

Rather than the centrosaur-like Monoclonius of my childhood, it looks like this fairly plain-looking ceratopsian grew up into something a bit more spectacular. But we'll need further study and, hopefully, more specimens to find out exactly what, and exactly how extreme, that transformation may have been.

* Ryan, M.J. (2006). "The status of the problematic taxon Monoclonius (Ornithischia: Ceratopsidae) and the recognition of adult-sized dinosaur taxa." Geological Society of America Abstracts with Programs, 38(4): 62.

Friday, November 2, 2012

The Flying Longipterygids

I started to get a little carried away in my previous post on longirostrisavisine tails, so I decided to split the finished post in half and use this one to delve a little more into the possible implications the odd tails and clawless wings of that group would have had on their flight styles.

As mentioned previously,  longirostravisines, unlike most other enantiornitheans, lacked claws on all three of their manual digits, a trait apparently acquired separately of the Carinatae (Ichthyornis + modern birds). In the last post I speculated that this might have reflected a distinct flying (or at least landing) style. But how much do we really know about longipterygid flight?

Fig. 10 from Close & Rayfield 2012, click to big it up. Note the three general clusters of continuous-flapping (red), soaring and flightless (yellow and gray), and bizarro enantiornithean style (green).

In their recent paper, Close & Rayfield attempted to correlate wishbone (furcula) shape with flight style. Many enantiornitheans in the analysis plotted together in a cluster well separated from modern birds, but close to basal avialans like Confuciusornis which are usually presumed to have been gliders. Oddly, in the Close & Rayfield figure reproduced above, Rapaxavis (no. 103), a longirostravisine, clusters with the weirdo enantiornithean-style fliers, while more basal longipterygid Longipteryx (no. 98) groups with continuous-flapping fliers and is marked as an ornithurine (something seems off here).

In another recent open-access paper on Mesozoic bird flight styles, Wang et. al (2011), using wing element and primary feather length ratios, found Longirostrisavis to be a continuous-flapping flier, and Longipteryx either a continuous-flapping or a flap-gliding flier, roughly the opposite result of the Close & Rayfield furcula-based analysis.

 The fact that two independent analyses using two distinct methods produced different results probably does not bode well for the precision of either method. Clearly, we need to figure out better methods to more reliably tests flight styles in extinct birds.

Wednesday, August 1, 2012

The Tail of Shanweiniao


Fossil tail feathers of S. cooperorum, from O'Connor et al., 2009.
As a follow-up to last month's post on the smallest Mesozoic theropods, here are a few additional observations on the small longipterygid Shanweiniao. Like other longirostravisines*, Shanweiniao cooperorum had reduced "hands" entirely lacking claws. This reduction of wing claws seems to have occurred independently of modern birds within this uniquely specialized group of enantiornitheans. (Euornitheans seem to have lost the bulk of their wing claws around the level of Carinatae, though many modern birds still retain at least keratinous claws on their wings, and longirostravisines may have as well).

S. cooperorum itself is most well-known for its elaborate tail made up of six ribbon-like feathers. Those feathers overlapped at the base, and may have acted as an air brake for precise landings with the feet on small branches. It's possible that most other enantiornitheans, which lacked long feathery tails and also retained wing claws, landed by simply smacking clumsily into tree trunks or brush and grabbing on with all four limbs.

Wednesday, July 25, 2012

Wrong for the Right Reasons

Outdated restoration of a Protoceratops andrewsi nesting
ground. Painting by Charles R. Knight, 1922.

Flipping through an old dinosaur book from the 1970s or early 1980s can be pretty fun. Nostalgia aside, it's great to see how far the science of paleontology has progressed in just a few decades, and also have a few laughs at the (from our modern perspective) outrageously outdated ideas and reconstructions we find. (David Orr's blog Love in the Time of Chasmosaurs has a great, long-running series covering "vintage dinosaur art" that lovingly pokes fun at some of the mistakes made by past palaeontographers.) Old dinosaur TV shows can be just as good. Last week, Mrs. M recorded a bunch of dinosaur shows for me which were airing on the Science Channel. I hadn't seen any of them before, and didn't realize until I hit play that I was in for a blast from the past. The shows were obviously old-school, narrated by Jeff Goldblum (I assumed these had come out around the time of The Lost World: Jurassic Park until one episode started discussing finds from later in the 1990s like Beipiaosaurus). One episode featured a segment on Roy Chapman Andrew's famous discovery of dinosaur eggs in the Gobi Desert, and the infamous misinterpretation of the eggs as belonging to Protoceratops rather than Oviraptor. This is just the kind of paleontological gaffe we paleo fans get schadenfreude out of today. After discussing the refuted hypothesis that an Oviraptor found on a nest of these eggs was first thought to be eating them rather than guarding them as later finds suggested, Mrs. M asked the obvious question: Why, given that this thing was found on top of the eggs, did they assume the eggs belonged to a different dinosaur?

Tuesday, June 5, 2012

The Smallest (Mesozoic) Theropods

The online community of paleontology fans seems to have an unnatural preoccupation with size. Visit any dino-related message board, and you will find near-daily debates over which carnivorous theropod was bigger (or more specifically, longer). Carcharodontosaurus? Giganotosaurus? Tyrannosaurus? Hint: if the length estimates are within a meter of each other, the weight estimates vary widely, and the beasts in question are known only from one or two fragmentary skeletons, the correct answer is "eh, they're all about the same size, give or take." Also, Therizinosaurus and Deinocheirus, being wimpy herbivores, definitely do not count.
Size comparison of select small non-pygostylian theropods.
From left: Palaeopteryx thompsoni, "Ornithomimus" minutus,
Parvicursor remotus, Epidexipteryx hui.
By Matt Martyniuk, licensed.
Less often, you may come across a discussion about which dinosaur was the smallest. These usually are not the heated debates you find with the mega-carnivores, but rather casual examination of minutiae and bringing up oft-forgotten species. Yes, everybody knows Compsognathus. But did you know the "chicken-sized" type specimen is a subadult or juvenile, and the referred French specimen is much larger? And anyway, Parvicursor was daintier by far. At 34cm (13in) long, Anchiornis was hailed as the smallest dinosaur when it was initially described, but subsequent specimens were larger (up to half a meter in length; still smaller than Compsognathus and slightly shorter than the ~40cm Parvicursor). Epidexipteryx, at a stubby, tail-free 25cm (10in) in length, was the shortest of them all, but its lack of a long tail means that it was a bit larger than the competition in mass. And anyway, isn't Epidexipteryx a bird?

Sunday, April 1, 2012

What Is Enantiornis?

Enantiornis leali was among the first enantiornithes to be found, and the first to be recognized as a member of a unique lineage of "opposite birds" separate from modern birds (Gobipteryx minuta, now recognized as an advanced enantiornithe, was found earlier). But despite being such a widely recognized and historically important member of its namesake group, little can actually be said about this species in terms of ecology or life appearance. Of course, that can't stop us from trying to figure out as much as we can by examining the available evidence and ecological context of these long-dead birds.

Monday, December 5, 2011

Waddle, _Achillobator_, Waddle!

Above: Revised illustration of Achillobator giganticus with corrected leg proportions. Scale bar = 500 mm. By Matt Martyniuk, all rights reserved.

"I've hunted most things that can hunt you, but the way these things move..."
"Fast for a biped?"
"Cheetah speed. Fifty, sixty miles an hour if they ever got out into the open, and they're astonishing jumpers."

This quote from the original Jurassic Park film did much to cement the image of dromaeosaurids, the raptor* dinosaurs, in the public consciousness as fleet-footed hyper predators. Despite being nearly 20 years old, this portrayal has by and large remained unchanged in popular culture, with raptors often stock monsters with near-supernatural murderous abilities in everything from tongue-in-cheek xkcd comics to (I hope) tongue-in-cheek made for SyFy movies.

*Yes, I'm going to commit a cardinal sin and refer to dromies as "raptors". "Raptor" in ornithology refers to most predatory birds, even those that hunt on the ground (the Raptor Research Foundation considers Secretarybirds to be raptors). Since dromaeosaurids were both predatory and birds under any sane definition of the word, there should be no problem referring to them as an extinct group of raptors.

But were raptors really particularly fast? Bipedal running speed in digitigrade animals (that is, those that walk on their toes like birds rather than their ankles like humans) is usually roughly determined by the ratio of the lower leg bones (the tibia/tibiotarsus) to the upper foot bones (the metatarsus). The longer the upper foot is in length compared to the lower leg, the faster an animal could run. Therefore, we would expect the fastest theropod dinosaurs to be those with the longest metatarsi relative to tibiae.

A prime example of a theropod specialized for running very very quickly are the parvicursorines. This specialized group of alvarezsaurids (strange theropodan insectivores with stout, powerful arms each bearing one very large claw) has among the longest lower leg to upper leg ratio of any Mesozoic dinosaur group.  Looking at the statistics compiled by Mickey Mortimer at The Theropod Database (a phenomenal resource I turn to so often I really should just make it my browser's home page), the type specimen of Parvicursor remotus (see leg diagram here) has a femur 52.6 mm long, a tibiotarsus about 75.6 mm long, and a metatarsus 58 mm long. The functional lower leg is 113 mm long, well over twice the length of the upper leg. More importantly, the lower leg and upper foot bones were fairly close to being equal in length. This animal was clearly a speed demon.

How does this compare to raptors? If, as Jurassic Park claimed, raptors were exceptionally fast, we would expect them to have similarly long lower legs. The terrifyingly human-sized raptors in JP were a Hollywood invention, but we do know of raptor species slightly smaller and slightly larger than they were.

On the smaller side were the famous Deinonychus antirrhopus. According to TTD, the femora of one relatively complete specimen measured 248 mm, with a tibia 324 mm long, and a metatarsus 151 mm long. Again, the total lower leg length is nearly double the upper leg. But the upper foot bones were only half as long as the lower leg bones.

The "fast raptor" meme was started by John Ostrom himself, when he first described Deinonychus in 1969. This was merely speculation on his part, as the hind limb was not completely known in the first specimens. Ostrom actually changed his opinion in later papers, finding that the femur was shorter than he'd initially thought, and that the foot bones were surprisingly short compared to other dinosaurs. Not only was Deinonychus not particularly fast, it probably could not have been nearly as fast as most other small theropods, including modern flightless birds, let alone cheetahs.

Another very popular type of raptors are advanced giant dromaeosaurines (Utahraptor and Achillobator). I recently found myself revising an older drawing of an Achillobator giganticus, which were, as mentioned above, only slightly larger than the Jurassic Park raptors. Many young dinosaur fans are very attached to these species in part because they're much larger than most other raptors, and because they had a slightly anthropomorphized novel written about them by Bob Bakker shortly after JP was released (Raptor Red). As a result, these big birds have a cachet in the collective consciousness similar to the generally more famous Deinonychus and Velociraptor--that of super-fast, agile and intelligent predators.

However, when finishing up my revised drawing, I had to double check the proportions several times to make sure I wasn't screwing it up. To my amazement, the legs, particularly the lower legs and upper foot bones, looked almost laughably short. Again according to TTD, the femur of A. giganticus measures 505 mm long, the tibia 490 mm long, and the metatarsus a paltry 234 mm long--less than half the length of the tibia. Not only is the metatarsus much, much shorter than the tibia, the entire lower leg in only marginally longer than the femur! The first thing that struck me wen looking at my own reconstruction was that this looked like the dromaeosaurid equivalent of Majungasaurus, those abilisaurids with the ludicrously short legs (which, coincidentally like Achillobator, have been suggested to be made up of chimeric specimens). It is also reminiscint of another stout-legged dromaeosaurid species, Balaur bondoc. While Balaur have been suggested to be possibly herbivorous due to these strange proportions, partial jaws and some teeth of Achillobator confirm that they were carnivores. But with legs like those, it's hard to imagine these creatures behaved the way the public imagines raptors to have done, chasing down fast moving prey. Frankly, it's hard to imagine Achillobator doing much beyond waddling across Nemegtian lake shores hunting turtles in epic slow-motion chases.

For the record, no described specimen of Utahraptor preserves both a femur, a tibia, and a metatarsus, so it's impossible to say whether or not they had the same squat proportions (unless somebody has some more detailed information on the numerous undescribed specimens in the BYU collections). For now, it would be safe to assume that they, too, would have been a laughing stock if they were caught trying to run.

Ok, but why would predatory animals have such stubby legs? There is a lot of evidence that dromaeosaurids were specialized for hunting big game, often animals larger than themselves. Deinonychus are infamous for their association with large ornithopods Tenontosaurus tilletti, and while evidence suggests they mainly targeted juveniles (Forster 1984), these were still much larger in terms of weight than even adult Deinonychus. Velociraptor are known to have grappled with the larger Protoceratops, and even a rumored specimen of a Microraptor apparently preserves evidence that they tackled prey larger than themselves. The short legs, especially the short foot bones, seem to be linked with the function of the large sickle-claw, making lack of speed a trade-off for improved ability to grapple and kill large game. Dinosaurs like Tenontosaurus and Protoceratops probably weren't particularly fast-moving themselves, making this sacrifice in speed worthwhile for the chance to down a massive animal that could provide a whole lot of food.

In the end, while the raptor chase scenes in Jurassic Park remain some of the most exciting parts of the movie, they require a significant amount of disbelief to be suspended; after all, it would be more realistic but slightly less suspenseful if Laura Dern had been able to evade the raptors in the power bunker by simply breaking into a light jog.

Friday, September 16, 2011

Feathers ARE Color

A lot of my posts lately have been dedicated to color in prehistoric feathers (primer here). As a  paleontographer, it's hard not to get excited about finding new ways to more accurately and naturally depict long-gone animals, and I know a lot of you reading this feel the same way. It can also be frustrating knowing the basic color palate we're dealing with, but having specific data from only a handful of species to draw inspiration from. I've already seen, not surprisingly, a few illustrations of Microraptor, Xiaotingia, etc. that basically mimic Anchiornis down to the spangles. We're so conditioned to follow phylogenetic bracketing that it's tempting to use what little info we have, and extrapolate it to close (and even not so close) relatives. This can apply to larger feather patterns as well; as I mentioned in this post, it's fine to extrapolate Microraptor-style feathering to Velociraptor, but it's not the ONLY way to do it, nor is it even necessarily the most plausible for a creature of such different size and ecosystem, as many online critics of Dinosaur Revolution would have you believe ;)

With that in mind, I want to start with a disclaimer: this kind of info only gets you so far. I'm not setting out to write the inerrant Bible of paleoart in these types of posts. Yes, all the evidence we have of dromaeosaurs shows full, lush feathering equivalent to small modern birds. But then again, we're dealing with small prehistoric birds here. Yes, we can interpret feather coloration and use inferences from modern birds and biochemistry to say what colors are likely and which are unlikely; but we can't always identify structural color in fossils, and we have yet to identify carotenoids, and many small dinosaurs we think of as "carnivorous" might well have trended more toward omnivory, insectivory, etc., or other unforeseeable pathways to those tasty, tasty bright yellow pigments.

Ok, preamble out of the way, the point of this post is to provide a general way I've used, and others can use, to try to make somewhat educated guesses about coloration in prehistoric birds which have not yet been analyzed for color pattern.

A few people pointed out to me when this recent paper by Wogelius et al. came out, in which the research team was able to identify color patterns in some Mesozoic birds using chemical markers rather than direct observation of melanosomes, that their reconstruction of Confuciusornis based on these findings was pretty similar to the restoration I'd done a while earlier.


Above: Restoration of Confuciusornis by Richard Hartley, from the press release. Below: My own earlier restoration of C. sanctus.


The two are pretty similar in the broad pattern: dark head, body, and coverts, white or light-colored wings with more black on the secondaries than the primaries. Now, so far this is only one data point, so I don't want to draw too many conclusions. But I was not simply guessing when I restored C. sanctus that way back in 2009.

The trick is to understand what you're looking at when you see a fossil feather. These are often referred to as 'impressions', but often the impressions are only part of the story, or even completely absent from the fossil. The breakthrough that led Vinther , Prum and others to figure out how to suss out feather color, was in realizing what fossil feathers are made of.

As Prum summarized on the Skeptics Guide to the Universe podcast a few years back, traditional wisdom held that the dark, 'carbonized' looking fossil feathers were the result of bacteria. Now, some old-school feather impressions, like those from Solnhoffen and the Santana formation, do contain nice, deep, actual impressions. These look very different from the stuff you find in the Jehol (compare the fossil feathers of the Berlin Archaeopteryx with the holotype of Microraptor gui). But most fossil feather,s including the famous single-feather holotype of Archaeopteryx and most Jehol stuff, are dark stains in the rock. Under the microscope, these looked to early researchers to be made up of fossil bacteria which had eaten away the feather keratin during decomposition.


Above: Photograph of an unsubscribed Anchiornis specimen by Robert Clark, from National Geographic, showing clear color patterns matching those predicted by Vinther et. al.

What Prum, Vinther, etc. showed in recent years is that this is flat-out wrong. Those granules are not bacteria--they're melanin! When you look at a fossil feather, most of the time, you're looking directly at the color pattern of the feather itself, the keratin and everything else having long since disappeared. This is especially apparent in very well-preserved fossils; for example, the beautifully preserved new Anchiornis specimen above is essentially proof of Vinther's hypothesis, which had previously been based on more obscured differences in shade. This is where my method of eyeballing it falls flat--I'd never have gotten the correct pattern from the specimen Vinther was looking at without really close physical examination. You need really nice specimens for it to conceivably work, or you have to Dave-Peters the heck out of low-res images trying to spot differences in contrast on the feathers.

Luckily, Confuciusornis was a safe bet, because so many specimens are known, and you can start to see patterns emerge. Many of the best specimens tend to have a very dark halo of feathers around the body and arms, with the wing feathers very faint, even sometimes difficult to see at all. Knowing that dark feathers means dense melanin = dark coloration, and light color = lack of melanin = light color, it was easy to come up with a good guesstimate of the life coloration. This was first inspired by Longrich's work on Sinosauropteryx, showing that the apparent bands in the tail were due to color patterning, which was later supported by published studies.

Obviously this is not a foolproof method. But it's a good place to start for artists who may want to add a little evidence-based thinking to their reconstructions, even if the evidence itself is wide open to interpretation. At the very least, if a good specimen has obvious areas of light and dark, I'd personally restore that pattern in a life illustration. It may end up being wrong, but it's better than pure speculation.


Monday, May 30, 2011

Know When To Fold 'Em


Above: Maximum wrist folding for the theropods studied by Sullivan et al. 2010. Not to scale.


(Cross-posted from Art Evolved)

To continue talking about aspects of maniraptoran anatomy that can be a bit vaguely defined in the minds of paleoartists, I'm going to write a bit on the issue of wrist folding. As most of you will know, a major characteristic of maniraptorans is the semi-lunate carpal, the half-moon shaped bone in the wrist that allows the blade of the hand (metacarpal 3) to fold backward toward the forearm (ulna). While this is common knowledge among paleo buffs and artists, what seems to be less understood is exactly how tightly the hand (and in aviremigians, the wing) could actually fold up. I myself have never been too clear on the issue, and there don't seem to be many papers addressing this. But in the last few years, a few papers have come along that can help shed light on the subject. The first was Senter 2006, which studied the full range of motion in the forelimbs of two dromaeosaurs, Deinonychus and Bambiraptor. The second was Sullivan et al. 2010, which examined the range of motion in the wrist of several species representing each major group of non-avialan maniraptorans.

Both papers, however, present geometric data that can come across as a bit inaccessible for your average artist, so I'm going to try to break down their conclusions for those of us who are more visual thinkers. The Sullivan paper, in particular, discusses the degree to which the wrist could fold, but doesn't necessarily provide diagrams or even final angle between the metacarpals and ulna for each species that could be used as a simple reference. I've done my best to translate their findings into the image at the top of this post, using modified skeletal diagrams by Scott Hartman and Jaime Headden.


Above: Anatomy of a maximally folded wing of the Wild Turkey Meleagris gallopavo, modified from Sullivan et al. 2010
The degree of wrist folding is controlled by two wrist bones. The cuneiform, on the inside where the wrist meets the bottom of the distal ulna, provides an inner limit. The cuneiform blocks the hand from actually touching the ulna. The radiale, on the outside of the fold, forms the surface which the wrist cannot fold beyond. This is basically a little process anchored to the tip of the radius where the top part of the hand articulates. The hand can obviously not fold beyond the angle of the radiale, or the animal would dislocate its wrist. Therefore, the angle the articular surface of the radiale forms with the ulna is used as the key factor in determining maximum wrist folding by Sullivan et al. Again, see my interpretation at the top for how their results likely translate into life position.
The results show that in almost all maniraptorans, the wrist could not be folded to the same degree as modern birds (for comparison, see the photo of the turkey wing above, which is at its own maximum folding point). Note that in actual, functional angle of folding in the turkey is 57 degrees between MCII (where the feathers attach) and the ulna. To see how this translates into a live animal, here's a photo of wild turkeys nicely showing the way the feathers fold (photo by D. Gordon E. Robertson, from Wikipedia, licensed):
The wrist is located about where the coverts form the point of a triangle, following the line formed by the border of the the brown secondary (ulna) feathers and white banded primary (metacarpus) feathers. Note that with the wrist folded at a 57 degree interior angle, the feathers (especially the secondaries, which help cover the primaries when folded) are basically stacked one on top of the other with little to no fanning out at the tips. This is because the feathers also have some ability to move at their bases, and can themselves fold relative to their anchor bones through muscle and ligament action.

Looking at the aviremigians in the diagram up top, it is apparent that their wrists could not fold tightly enough to fold the wing feathers to the same degree as a modern turkey. Small deinonychosaurs like Sinovenator and Bambiraptor could achieve close to a 100 degree angle (see image of Bambiraptor wing folding above, from Senter 2006), but larger ones like Deinonychus seem to have lost some of that folding ability, presumably for increased use of the forelimbs in predation. Indeed, if Deinonychus retained long remiges, they would hardly have been able to fold at all, and would have been permanently fanned out (not that this would have gotten in the way of grabbing prey, as Senter pointed out). This lack of ability to tightly fold the wrists may have posed a significant problem for those species with very long remiges, like Microraptor gui. Dave Hone, who was a co-author of the Sullivan paper, discussed alternative ways they could have kept their remiges free of the ground at his blog last year.

In pygostylians, the degree of wrist folding began to approach that found in modern birds. Eoconfuciusornis, for example, could fold its wing to about the same degree as a turkey. Where it gets weird is in the oviraptorosaurs. As I mentioned in my post on the Ashdown maniraptoran, oviraptorosaurs (at least the small basal ones like Caudipteryx) seem to have been capable of folding their wings far beyond what is possible for even many modern birds. It's unclear why this is so, especially as the remiges of Caudipteryx, while clearly for display, are not exactly very long compared to the body. Certainly its wings were much smaller than those of paravians, which would have presumably had more need to fold them up. I've seen this mentioned as possible evidence in support of the hypothesis that oviraptorosaurs are in fact avialans, and that the extreme folding of the wrist was inherited from flying ancestors, though I can't think of where. Sullivan et al. do note that more than folding up the remiges to keep them safe from wear and tear, wing folding is an important part of the avian flight stroke, and it makes sense that it would have become more developed in flying forms.

Anyway, we've only got a handful of specimens that have been specifically studied in regards to the degree of wrist folding, and there may well be exceptions in each maniraptoran group, where certain lineages independently evolved a greater or lesser degree of wrist folding from their ancestors as seems to have happened in therizinosaurs, where the derived Alxasaurus can fold its wrist more than the basal Falcarius, and deinonychosaurs, where the relatively derived Deinonychus can fold its wrist less than the more basal Bambiraptor. So this guide shouldn't be considered as a set of hard and fast rules, but rather a starting point for artists who want to make their restorations as plausible as possible.

Finally, a few days ago I posted a teaser for this post challenging people to determine what aspect of the above Deinonychus illustration was incorrect. By now it should be clear that the wrist is folded too far back. Appropriately enough, the first one to nail it was the artist, Nobu Tamura, himself! Commenter A.G. came close, speculating that it was due to the orientation of the glenoid, but that has more to do with the range of motion of the upper arm and how far it could extend into a bird-like flapping position, rather than the way the wing folds up. Good job guys!

References
* Senter, P. (2006). "Comparison of Forelimb Function Between Deinonychus And Bambiraptor (Theropoda: Dromaeosauridae)". Journal of Vertebrate Paleontology, 26(4): 897–906.
* Sullivan, C., Hone, D.W.E., Xu, X. and Zhang, F. (2010). "The asymmetry of the carpal joint and the evolution of wing folding in maniraptoran theropod dinosaurs." Proceedings of the Royal Society B, 277(1690): 2027–2033.

Tuesday, May 17, 2011

Tyrannosaur Tooth Count

Making the rounds right now in the media is a story about a newly described, well-preserved baby Tarbosaurus bataar that helps shed some light on the way tyrannosaurs grow, as well as touches on lingering controversies. Plenty of other blogs have already covered this, so here's a link to the backstory from Brian Switek at Dinosaur Tracking.

Interestingly, the baby Tarb has 15 teeth in the lower jaw, the same number as adult T. bataar. There has been controversy over whether or not tyrannosaurs reduced their number of teeth as they grew, particularly when it comes to the controversial taxon Nanotyrannus lancensis. Nano is known from two specimens (one is nicknamed "Jane") that, depending who you talk to, might really be simply juvenile specimens of the contemporary Tyrannosaurus rex. The differences cited to separate the two boil down to differences in the braincase (certain braincase changes were demonstrated in the new juvenile Tarbosaurus as well), and the number of teeth. Adult T. rex are usually said to have only about 12 teeth in the dentary, while specimens of N. lancensis have a whopping 17. The new juvenile Tarb suggests that in at least some tyrannosaurs, the tooth count is not drastically reduced during growth from juvenile to adult. However, as the authors caution, this same pattern may not necessarily hold true for other tyrannosaurs, even very close relatives.

And, the same pattern does not hold true for the very closely related T. rex. Also making the blog rounds these last few days has been this video of Jack Horner's talk at TEDx in Vancouver (thanks to David Orr at Love in the Time of Chasmosaurs for posting the video link!).


Here Horner gives the basics of his theory that dinosaurs are oversplit, not in the subjective taxonomic sense, but in the more objective biological sense that specimens that could be shown to belong to one species actually represent juveniles of other species. You've all heard the details before, but towards the end he shows a slide (reproduced above) that is pretty damning to the crowd who support the validity of N. lancensis. In fact, adult specimens of T. rex show a very wide ranging tooth count, and it even appears to correspond with relative size (and presumably growth stage. If anything, the number of teeth seen in N. lancensis specimens are only one or two teeth outside the range of variation for T. rex proper, a minor variant that can almost certainly be attributed to ontogeny, and not some cryptic species of giant tyrannosaur lurking in the Lancian faunas that has so far only been identified by two juvenile specimens, while the very common T. rex is known from no juveniles at all.

Anybody know the tooth count for the "Tinker" specimen, currently held in a private collection?

Monday, May 16, 2011

Confuciusornis: Bird-o-Dactyl


There's been a lot of debate about Confuciusornis lately. Could it fly? If so, how? And how well? It probably wasn't doing anything like a modern bird does. Studies of its feather strength suggest it couldn't do more than glide (or could it?). But studies of its forelimb and shoulder girdle show it couldn't lift its arm much above the horizontal plane, making flapping pretty much impossible. Unless that huge, fenestrated deltopectoral crest gave it a rather unique flight stroke that only minimally involved the humerus.

Or, maybe this was a small theropod with enormous, high-aspect ratio wings larger than those of any other early bird, with asymmetrical feathers, puny feet and short legs ill suited for running and a small, barely reversed hallux ill suited for climbing, which couldn't flap and could barely glide with its thin feather shafts, yet is consistently found preserved as enormous flocks at the bottom of deep lake deposits. In which case the giant wings would be for display, obviously, to hopefully impress a predator so much that they decline to eat the poor bird which has no means of escape or defense other than to flee into the depths of the water like a 1960s brontosaur, only to remember that it also can't swim. No wonder they're extinct! Anyway... I hope much, much more study (and some wind tunnel tests) will eventually help untangle this mystery. For now, I was struck by something a little more frivolous. Working on a lateral view of Confuciusornis sanctus, checking and re-checking papers to make sure proportions are right, it started to look unmistakably like the profile of a... rhamphorhynchid pterosaur? Between this, and basal paravians with expanded, diamond-shaped vanes on the tips of their tails, in terms of general body plan there are some curious similarities (convergences?) between the first gliding/flying birds and primitive, long-tailed, high-aspect ratio-winged pterosaurs. My PhyloPic style silhouette version above.

Monday, February 14, 2011

Heat, Feathers, and Half-Arsed Velociraptor

Above: Comparison of common Velociraptor reconstructions by artist Tomozaurus, used with permission.

A month or so ago, this diagram (also shown above) produced by an artist known as Tomozaurus stirred up a good deal of debate over at DinoForum. Tom was trying to illustrate common misconceptions about the most likely life appearance of dromaeosaurids. By now, everyone (including the birds-are-not-dinosaurs crowd) agree that dromaeosaurids were fully feathered and pretty bird-like. Whether or not to consider them actual birds is a matter of semantics at this point. But, among dino-fans weaned on their depictions in pop-culture, there seem to be a lot of heated reactions to depicting them as too bird-like. Many will admit that they had feathers, but stop short at reconstructing them in a really bird-like manner, preferring a short, cat-like pelt that allows the graceful and well-known contours of the skeleton to show through in life. But compare any bird skeleton to a live specimen, even those with "simple" feathers like chicks or kiwi, and you'll immediately see that this is the wrong way to go. Even most feathered theropod fossils show a feather covering that does not hug the body contours, but like modern birds, consists of a lot of poofy, long feathers (especially at the breast and neck) that would make them look very "bulky."

The debate about the above image concerned how well these principles should apply to larger dino-birds like Velociraptor. Velociraptor is perhaps the worst offender in this area due to its enormous popularity: it has a very well-ingrained image in the popular consciousness that, in all likelihood, doesn't match how it would have appeared in life. But just how likely is any reconstruction?

The fact is, we don't know very much at all about the feathering in Velociraptor. At least one specimen preserves quill knobs on the ulnae where large secondary feathers must have attached, so we know for a fact that it had wings. But what about the body feathers? Tom's picture supposes that we would do best to reconstruct the remaining feathers based on related (but much smaller) species in which the full compliment of feathers has been preserved; things like Microraptor, Anchironis, Archaeopteryx, and the unnamed species nicknamed "Dave". Based on these, Tom gave his "correct" Velociraptor a full set of long primary feathers (present in Micro and Archie but much shorter in Dave and Anchi), a feather crown (present in Micro and Anchi but not Dave and Archie), flight feathers on the hind legs (present in Micro, Anchi and Dave but not Archie, though the last does have "bell bottoms" of long, non-planar pennaceous feathers down to the ankles), and feathers covering the face and most of the snout (present in all but possibly Archie). Last, he restored the body contour feathers as pennaceous rather than downy. This is the most problematic, present (apparently) in Anchiornis but not in the others (Archaeopteryx has pennaceous feathers over the hips but this appears to be a single or paired feather tracts (pterylae), and the rest of the body is covered in plumulaceous feathers or simple protofeathers).

In contrast, Tom presents two "incorrect" versions: the Greyhound/Lizard (which is so obviously wrong there's not much else to say about it) and the "Half-Arse." The later is interesting because while it deviates considerably from the inferences drawn based on its relatives, there's nothing obviously inaccurate about it, or at least implausible. The drawing seems to be identical to the Velociraptor computer models used in the TV show Dinosaur Planet: feathered, but barely so, with a short, mammal-like pelt hugging the contours of the body, a large crown for display, and many featherless areas of the body.

Defenders (or at least devils advocates) for this reconstruction pointed out that it doesn't deviate too wildly from larger, flightless modern birds. Ostriches (Struthio camelus) are famously stripped-down of feathers, more so than many people think (see image above, showing the naked underside of the wings and featherless torso). However, ostirches are also quite a bit larger than Velociraptor, and smaller ground birds from the same environment like the Secretary Bird (Sagittarius sepentarius) lack extensive naked patches. On the other hand, Rhea (Rhea spp.), which are similar to Velociraptor in weight, do have naked patches on their underwings, though not as extensive as ostirches (see image below).

So, while I still think the rather short body feathers would be a little far-fetched (longer ones would be better for thermoregulation--if overheating is the issue, the feathers would probably simply be lost entirely, which is not the case in modern birds that lose feathers only on extremities), the Half-Arse version doesn't seem all that bad.

But there's more that needs to be taken into account. A great post at Tetrapod Zoology today touches on some aspects of featherless patches on birds and its effects on thermoregulation. A bit counter-intuitively, a heavy feather coat can actually help keep birds cool--they're general insulators, not simply heat-trappers, like a thermos. In the post, Darren Naish discusses male wild turkeys, which famously have bare heads with brightly colored, outlandish soft tissue structures for display. This actually puts the male birds at a disadvantage, because all that bare skin causes the males to be more prone to overheating, requiring them to spend more time cooling in the shade than females. Like the tail of a peafowl, the naked heads of turkeys are a sexual display structure that puts the birds at a disadvantage when it comes to survival. Granted, this is only the example of one bird. I don't know how this might apply to, say, ostriches. Ostriches, like Velociraptor, inhabit a hot, arid environment. Indications suggest that Velociraptor lived in an even more desert-like setting, dominated by barren dune fields, making it a solidly desert bird. Would the extensive bare patches of the Half-Arse be beneficial in this setting, or would they tend to drastically overheat the animal under an unrelenting desert sun with few sources of shade?

Above: Photo of a Greater Rhea (Rhea americana) by Ramon Moller Jansen. This species is about the same size as an adult Velociraptor mongoliensis, but live in more lush environments with some tall shade plants.

According to Willmer, Stone & Johnson (2000), many ratites use similar strategies to regulate their body temperature and prevent overheating. Ratites such as the Rhea store their heat while active, and only actively attempt to shed it while at rest. This is achieved through strategies such as panting, drooping the wings (allowing air to conduct heat from the sparsely feathered underwings while at the same time shading them), and raising or lowering the sparse feathers of the back (known as ptilo-erection). It's interesting to note that in Archaeopteryx, the back is the only region of the body that has pennaceous feathers, better for trapping or shedding heat. With all of these adaptations, ostriches rarely have to seek shade, even when it's available (Levy et al., 1990). So while feather-loss in modern birds is an important strategy for those living in hot, arid climates, note that the pattern of loss is not random or extensive, but rather strategic, allowing for maximum thermal regulation.

If I were to speculate, I'd make an educated guess that bare patches in Velociraptor must have been limited to the legs, flanks and underwings for these reasons. Those areas could be shaded simply by the animals own body and cooled easily as needed. The head and neck would have been most prone to overheating. The animal could only shade these by adapting a Mei long style sheltered posture with the head tucked under the wing and body feathers (but only if a hefty body covering was present, not a form-fitting pelt). One question I can't seem to find an answer to is how ostriches cope with direct sun to their nearly bare heads and necks--the problem faced by male turkeys. My wild guess would be that the heads of turkeys are highly decorated with thickened skin, presumably a better insulator than the plain skin of an ostrich, which would allow more loss of heat to the air. Or maybe they bury their heads in the sand to keep cool... (I kid, I kid!). If anybody knows of any studies or physiological issues that would cause this to be a problem for one and not the other, please leave a comment!

References:
* Levy, A., Perelman, B., Grevenbroek, M.V., Creveld, C.V., Agbaria, R. and Yagil, R. (1990). "Effect of water restriction on renal function in ostriches (Struthio camelus)." Avian Pathology, 19: 385-393.
* Willmer, P., Stone, G. and Johnston, I.A. (2000). Environmental Physiology of Animals. Wiley-Blackwell, Science. 644 pp.

Monday, January 17, 2011

Theropods That Fit the Bill

[Image: Skull of a gull compared to a living specimen. The apparent differences in the extent of the beak are caused by the presence of different kinds of rhamphotheca.]

One aspect of Mesozoic birds and other theropods that doesn't get discussed much are their bills. Beaks or beak-like structures (generally, rhamphotheca) have a wide but extremely spotty distribution among Mesozoic theropods, and numerous theropod groups seem to have evolved them independently of one another.

Perhaps the most basal known theropod that likely bore a beak (assuming we can safely exclude the skull material attributed to the infamous "first bird" Protoavis) is Limusaurus inextricabilis from the Oxfordian, about 160 million years ago. Though it belonged to the otherwise toothy clade Ceratosauria, Limusaurus was completely toothless. To be precise, most theropods have teeth in the three major sections of their jaws: the premaxilla at the front of the skull, the maxilla behind it, and the dentary, or lower jaw. Ornithischian dinosaurs had an additional bone, the predentary, at the tip of the lower jaw that was always toothless, indicating that almost all ornithischians probably bore a beak, at least on the lower jaw (and ceratopsians added an additional, pre-premaxilla: the rostral). Limusaurus lacked teeth in the premaxilla, maxilla, and dentary, so it was completely toothless and, therefore, it is assumed to have been beaked.

[Image: Skull reconstruction of Limusaurus, posted by Dave Hone at his Archosaur Musings blog.]

As far as I know, Limusaurus is the only non-coelurosaurian theropod that bore a beak. Generally, this fits well with the idea that non-coelurosaurian theropods were hypercarnivorous flesh eaters with little variation in their diets. However, as a number of recent papers by Lindsay Zanno and colleagues has shown, coelurosaurs started playing around with omnivory and herbivory, and as a consequence, many lineages cast off some or all the sharp teeth that characterized their ancestors.

[Image: Skull reconstruction of Pelecanimimus by Ville Sinkkonen]

The first coelurosaur lineage to start shedding their teeth permanently were the ornithomimosaurs. This group is well-known for their toothlessness, and evidence from specimens with preserved keratin sheaths on the jaws (Norell et al, 2001) show definitively that they bore keratinous beaks on both the upper and lower jaws, at least in advanced species. As expected, the most primitive ornithomimosaurs still retained teeth. Pelecanimimus polydon, as its name implies, had teeth in the premaxilla, maxilla and dentary. The next most advanced ornithomimosaur, Harpymimus, is the first example among theropods of the "half beak." While its upper jaw was toothless and likely beaked, it retained teeth in the lower jaw. I'll come back to the implications of these "half beaks" further down. The most basal ornithomimosaur wich lacked teeth completely seems to be Garudimimus, though the status of Beishanlong is unknown.

After the ornithomimosaurs, beaks are found in therizinosaurs. Again, early forms like Falcarius had a full compliment of teeth, but in laker ones like Beipiaosaurus, the teeth became restricted to the middle of the jaws, leaving room for a beak in the front, similar to ornithischians. Next, oviraptorosaurs seem to have developed beaks fairly early in their evolution. While Incisivosaurus had teeth in both jaws (though restricted to the tips), Caudipteryx had only a few teeth in the premaxilla, another example of a "half beak" where a toothless lower jaw is matched with a toothy upper jaw. While the several possible intermediate forms lack skulls, both caenagnathids and oviraptorids proper had fully toothless jaws, so presumably they were fully beaked by the time they diverged.

Next up were the deinonychosaurs, and while some seem to have dabbled in omnivory, they were mainly carnivorous, and none seem to have developed beaks. Greg Paul is infamous for restoring them with cornified tissue or "proto beaks" at the tips of their jaws adjacent to teeth, but there isn't much evidence to support this idea as far as I know. However, many deinonychosaurs which preserve feathers show a (usually small) portion near the tip of the snout that is unfeathered. This featherless snout tip is also seen in some toothed, presumably beakless enantiornithines. It's possible this could be evidence of "rhamphotheca" in its loosest sense--the very lightly cornifies, flexible bill skin found toward the back of the beaks in some modern birds, where the horn-like, kerationous portion thins out into normal skin. More on these flexi-bills down the page.

[Image: My own simplified cladogram of Aviremigia showing some notable occurrences of beaked and half-beaked and beak-free birds. Excuse the quality in close-up, some of these were yoinked from works in progress.]

Around the base of Avialae, the occurrence of half-beaks seems to explode. Almost all known basal, non-pygostylian avialans lack teeth in the upper jaw (e.g. Jeholornis, Yandangornis) or lower jaw (omnivoropterygids) and, possibly, both (Jixiangornis preserves no teeth and may have been full-beaked, but the skull is badly crushed, and crushing has been known to obscure the tiny teeth that should be present in other basal avialan specimens). This trend appears to culminate with the confuciusornithids, which are not only toothless but have sharply pointed jaws that, in some very rare specimens, preserve the actual keratin of the beak. These impressions show that even in these fully beaked birds, the rhamphotheca was thin and delicate and probably not as heavily mineralized as in modern birds.

The next bit is rather odd given the trends seen at the base of avialae. In most basal ornithothoraces (the group that includes enantiornithines and ornithuromorphs), the jaws are fully toothed, with no evidence for beaks. It's tempting to think that this could unite the enantiornithines with the toothy, beakless deinonychosaurs and Archaeopteryx in a "Sauriurae" to the exclusion of the beaked birds. However, given the numerous times beaks have evolved independently in vertebrates, it's not unthinkable that each of the half-beak examples above arose independently of one another (or, that some reversal occurred at the base of ornithothoraces to return birds to a state of fully-toothed maws). Either way, while many enantiornithines preserve jaw material, only a few exhibit the kind of toothlessness at the front of the jaws that could imply a beak. These include the half-beaked Alethoalaornis (with a toothless dentary but toothed premaxilla), the fully-beaked Gobipteryx, and the half-beaked Boluochia. Boluochia had teeth in the dentary but none in the upper jaw and, in fat, had a strongly hooked premaxilla similar to the hooked beaks of modern raptors. Enantiornithine relationships are too unresolved to be able to tell if these beaked birds all form a natural group, or if beaks evolved multiple times among enantiornithes, but given their diversity it's a safe bet that many different lineages came up with their own particular feeding solutions.

[Image: The compound rhamphotheca of an albatross is visible as distinct sutures, and is also found in some non-avian birds. Image from the RSPB.]

As expected based on the enantiornithine record, most primitive ornithuromorphs (the fan-tailed birds, including Aves) either lakced beaks or exhibited a half-beaked configuration. While Hongshanornis was originally reported to have a beak, Jingmai O'Connor and colleagues later showed that it had tooth sockets preserved in the upper and possibly lower jaws (same goes for the related Longicrusavis). The earliest fully-beaked ornithuromorph is also one of the most primitive, however: Archaeorhynchus lacked teeth and had a flattened, Spoonbill-like beak. The songlingornithids (such as Yixianornis), and the later hesperornithines and Ichthyornis all had a therizinosaur-like configuration, with toothless premaxilla (and even predentary-like bones in the hesperornithines) with toothy maxilla and dentaries. Evidence from bone texture shows that likely had keratinous beaks at the tips of their jaws, and either feathery toothed jaws or pliable, skin-like rhamphotheca further back. Since both major lineages of avians lack teeth, it's likely their common ancestor was also fully beaked, so teeth must have been lost for good in the bird lineage shortly after Ichthyornis diverged. Interestingly, studies of ichthyornithines and hesperornithine bone structure shows that they likely had "compound rhamphotheca", and this may have been the ancestral condition for modern birds (Heironymous & Witmer, 2010). While the quintessential bird beak is made up of a single keratin sheet covering the jaw, in species with compound beaks, the keratin is arranged in discrete plates on the jaws. This can best be seen in some modern seabirds like the Albatross.

Unfortunately, in interesting taxa like Hollanda, Gansus, and Patagopteryx, the condition is unknown. However, we can use parsimony and phylogenetic bracketing to try and come to a reasonable guess. Most studies find these three to be ornithuromorphs more primitive than the hesperornithines and Ichthyornis. Given the condition in Ichthyornis, it's most likely that Archaeorhynchus evolved its toothless beak independently of more advanced birds, most of which have toothed upper and lower jaws with beaked tips in the grade between Archaeorhynchus and Aves. While the three intermediate birds may well have lost some or all of their teeth independently again, it's probably more parsimonious to assume that like hesperornithids, hongshanornithids and songlingornithids, they were either fully toothed or had beaks restricted to the tips of the jaws.

[Image: Cassowary chick by Michael Thirnbeck, from Flickr. Note the horny beak only covers the tip of the bill, leaving the nostril surrounded by more skin-like tissue. Thanks to meidamon over at DinoForum for finding this and other pictures illustrating beak anatomy.]

So, to rephrase an old fallacy, what use is half a beak? Many Mesozoic coelurosaurs had teeth only on the upper or lower jaw, and most researchers have assumed that edentulous = beaked (see for example Zanno et al., 2009). But "beaks" are more complex than simple sheathes of keratin covering toothless parts of the jaw. As anatomist Larry Witmer has explained (in print as well as on the DML), rhamphotheca can consist of everything from solid, hard keratin (which, obviously, is a bit antithetical to tooth growth and replacement) to softer, pliable, barely mineralized tissue. For example, it's a general rule of thumb that the keratin rhamphotheca never completely encloses the external nares, meaning the nostrils of a bird are never encased in keratin. This is most obvious in species that have a cere, a prominent fleshy part of the posterior rhamphotheca found in pigeons, parrots and hawks, among other birds. But in many other birds (especially aquatic forms like ducks and gulls), the nostrils do appear to erupt from mid-bill. What's going on?

[Image: Duck skull by ~Oryx gazella~, from Flickr. Note that only the tip is fully keratinized.]

Basically, the "beak" of a duck (and many other birds) is only really solid towards the tip. The broad bill of a duck is, laterally, fairly soft, and made of rhamphotheca that is only lightly mineralized. Essentially, it's mostly toughened skin (this is why ducks and other anseriforms are particularly prone to bill injuries). In the kiwi, the nostrils don't just erupt from the "beak", they occur at the very tip. Again, the bill of a kiwi is not highly keratinized, but rather made up of soft, pliable integument full of sensory organs (Martin et al., 2007).

So, our mysterious half-beaked birds may have had some cere-like tissue covering the upper portion of the toothed bill, while the lower portion contained more keratinized rhamphotheca. Perhaps the upper jaw had a small keratinized tip wedged between the front teeth, as seen in toothed pterosaurs like Rhamphorhynchus and Pterodactylus. Or maybe the half-beaks of some of these birds contained little to no keratin at all. As the kiwi shows, it's not always necessary for all food-aquisition behaviors to have a beak or teeth.

Hopefully, this rough guide can also serve as a reference for artists, many of whom are a bit over-eager to add a beak to anything that is called a "bird." While a wide range of rhamphotheca like structures may have been present on Mesozoic birds, it wasn't necessarily present on all of them, and many probably looked a bit strange compared to the simple, smooth yellow bills of modern birds.

References
* Heironymous, L. and Witmer, L.M. (2010). "Homology and Evolution of Avian Compound Rhamphothecae." The Auk, 127(3): 590-604. doi: 10.1525/auk.2010.09122
doi: 10.1525/auk.2010.09122
* Martin, G.R., Wilson, K.-J., Wild, J.M., Parsons, S., Kubke, M.F., et al. (2007). "Kiwi Forego Vision in the Guidance of Their Nocturnal Activities." PLoS ONE, 2(2): e198. doi: 10.1371/journal.pone.0000198
* Zanno, L.E., Gillette, D.D., Albright, L.B., and Titus, A.L. (2009). "A new North American therizinosaurid and the role of herbivory in 'predatory' dinosaur evolution." Proceedings of the Royal Society B, 276(1672): 3505–3511. doi: 10.1098/rspb.2009.1029.